Investigation of Disease-Relevant Lysine Acetylation Sites in α-Synuclein Enabled by Non-canonical Amino Acid Mutagenesis
Curation statements for this article:-
Curated by eLife

eLife Assessment
This important work provides new insights into the role of lysine acetylation of alpha-synuclein, the protein involved in Parkinson's Disease. The evidence is convincing and the work will be of interest to researchers in the fields of protein biophysics and post-translational modifications.
This article has been Reviewed by the following groups
Listed in
- Evaluated articles (eLife)
Abstract
Aggregates of α-synuclein (αS) are hallmarks of synucleinopathies, including Parkinson’s Disease (PD) and Multiple System Atrophy (MSA). We have recently shown that αS lysine acetylation in the soluble monomer pool varies between healthy controls, PD, and MSA patients. We used non-canonical amino acid (ncAA) mutagenesis to express and purify all 12 currently known disease-relevant variants of αS and studied their binding to membranes as well as their aggregation propensities. We found that acetylation of lysine 12, 43, and 80 had particularly strong effects. To understand the implications for acetylation of monomeric αS found in healthy cells, we performed NMR experiments to study protein conformation and fluorescence correlation spectroscopy experiments to quantify lipid binding. We also investigated the effects of acetylation at lysine 12, 43, and 80 on fibril seeding in neurons. Collectively, our biochemical and cell biological investigations indicated that acetylation of K80 could inhibit aggregation without conferring negative effects on monomer function in healthy cells. Therefore, we studied the structures of fibrils with K80 acetylation through cryo-electron microscopy to uncover the structural basis for these effects. Finally, we identified inhibition of HDAC8 as a way of potentially increasing acetylation at K80 and other inhibitory sites for therapeutic benefit.
Article activity feed
-

eLife Assessment
This important work provides new insights into the role of lysine acetylation of alpha-synuclein, the protein involved in Parkinson's Disease. The evidence is convincing and the work will be of interest to researchers in the fields of protein biophysics and post-translational modifications.
-
Reviewer #1 (Public review):
[Editors' note: the authors have revised the work in response to the original reviews.]
Summary:
This paper describes experiments with alpha-synuclein (aS) with acetylated lysines (acK) at various positions. Their findings on how to use non-canonical amino acid (ncAA) mutagenesis to generate aS with acetylated lysines are valuable. The paper then continues with a range of experiments to characterise the acetylated alpha-synuclein constructs at different positions, with the aim of providing insights into which sites are relevant to disease or their function inside cells. The paper concludes these experiments with the suggestion that inhibiting the Zn2+-dependent histone deacetylase HDAC8 to potentially increase acetylation at lysine 80 may have therapeutic benefit. However, the relevance of most of these …
Reviewer #1 (Public review):
[Editors' note: the authors have revised the work in response to the original reviews.]
Summary:
This paper describes experiments with alpha-synuclein (aS) with acetylated lysines (acK) at various positions. Their findings on how to use non-canonical amino acid (ncAA) mutagenesis to generate aS with acetylated lysines are valuable. The paper then continues with a range of experiments to characterise the acetylated alpha-synuclein constructs at different positions, with the aim of providing insights into which sites are relevant to disease or their function inside cells. The paper concludes these experiments with the suggestion that inhibiting the Zn2+-dependent histone deacetylase HDAC8 to potentially increase acetylation at lysine 80 may have therapeutic benefit. However, the relevance of most of these experiments is unclear, mainly as the filaments that form from these constructs are different from those observed in human disease (but see below for more details). Moreover, using the recombinantly produced acetylated versions of alpha-synuclein to normalise mass-spectrometry data, the authors themselves report that acetylation of alpha-synuclein does not differ between individuals with Parkinson's disease or healthy controls.
Strengths:
The authors report difficulties with chemical synthesis and then decide to make these constructs using non-canonical amino acid (ncAA) mutagenesis, which seems to work reasonably well (yields vary somewhat). In the Conclusion section, the authors report that they used these recombinant proteins to obtain quantitative insights into the levels of acetylation of lysines in individuals with PD versus healthy controls, for which they find no significant differences. This part of the work is valuable.
Weaknesses:
The authors then use circular dichroism to show that aSyn with acK at position 43 has less alpha-helical content. From this result, they deduce that "only this site could potentially perturb aS function in neurotransmitter trafficking", but no experiments on neurotransmitter trafficking were performed.
-
Reviewer #2 (Public review):
Summary:
Shimogawa et al. studied the effect of lysine acetylation at different sites in the alpha-synuclein (aS) sequence on the protein-membrane affinity, seeding capacity in the test tube and in cells, and on the structure of fibrils, using a range of biophysical methods. They use non-canonical amino acid (ncAA) mutagenesis to prepare aS lysine acetylated variant at different sites.
Strengths:
The major strength of this paper is the approach used for the production of site-specific lysine acetylated variants of aS using ncAA mutagenesis, as well as the combination of a range of biophysical methods together with cellular assays and structure biology to decipher the effect of lysine acetylation on aS-membrane binding, seeding propensity, and fibril structure. This approach allowed the author to find that …
Reviewer #2 (Public review):
Summary:
Shimogawa et al. studied the effect of lysine acetylation at different sites in the alpha-synuclein (aS) sequence on the protein-membrane affinity, seeding capacity in the test tube and in cells, and on the structure of fibrils, using a range of biophysical methods. They use non-canonical amino acid (ncAA) mutagenesis to prepare aS lysine acetylated variant at different sites.
Strengths:
The major strength of this paper is the approach used for the production of site-specific lysine acetylated variants of aS using ncAA mutagenesis, as well as the combination of a range of biophysical methods together with cellular assays and structure biology to decipher the effect of lysine acetylation on aS-membrane binding, seeding propensity, and fibril structure. This approach allowed the author to find that lysine acetylation at positions 12, 43, and 80 led to lower seeding capacity of aS in the test tube and in cells, but only acetylation at lysine 80 did not affect aS-membrane interaction. These results suggest that lysine acetylation at position 80 may be protective against aggregation without perturbing the proposed functional role of aS in synaptic plasticity.
Weaknesses:
SDS is not a good membrane model to investigate the effect of lysine acetylation on aS membrane-binding because it is a harsh detergent and solubilizes membranes. Negatively charged vesicles or vesicles made of a mixture of lipids mimicking the lipid composition of synaptic vesicles are more accepted in the field to study aS-membrane interactions. The authors used such vesicles for the FCS experiments, and they could be used for the initial screening of the 12 lysine acetylated variants of aS.
-
Reviewer #3 (Public review):
Shimogawa et al. describe the generation of acetylated aSyn variants by genetic code expansion to elucidate effects on vesicle binding, aggregation, and seeding effects. The authors compared a semi-synthetic approach to obtain acetylated aSyn variants with genetic code expansion and concluded that the latter was more efficient in generating all 12 variants studied here, despite the low yields for some of them. Selected acetylated variants were used in advanced NMR, FCS, and cryo-EM experiments to elucidate structural and functional changes caused by acetylation of aSyn. Finally, site-specific differences in deacetylation by HDAC 8 were identified.
The study is of high scientific quality, and the results are convincingly supported by the experimental data provided. The challenges the authors report regarding …
Reviewer #3 (Public review):
Shimogawa et al. describe the generation of acetylated aSyn variants by genetic code expansion to elucidate effects on vesicle binding, aggregation, and seeding effects. The authors compared a semi-synthetic approach to obtain acetylated aSyn variants with genetic code expansion and concluded that the latter was more efficient in generating all 12 variants studied here, despite the low yields for some of them. Selected acetylated variants were used in advanced NMR, FCS, and cryo-EM experiments to elucidate structural and functional changes caused by acetylation of aSyn. Finally, site-specific differences in deacetylation by HDAC 8 were identified.
The study is of high scientific quality, and the results are convincingly supported by the experimental data provided. The challenges the authors report regarding semi-synthetic access to aSyn are somewhat surprising, as this protein has been made by a variety of different semi-synthesis strategies in satisfactory yields and without similar problems being reported.
The role of PTMs such as acetylation in neurodegenerative diseases is of high relevance for the field, and a particular strength of this study is the use of authentic acetylated aSyn instead of acetylation-mimicking mutations. The finding that certain lysine acetylations can slow down aggregation even when present only at 10-25% of total aSyn is exciting and bears some potential for diagnostics and therapeutic intervention.
-
Author response:
The following is the authors’ response to the original reviews.
Public Reviews:
Reviewer #1 (Public review):
Weaknesses:
The authors then use circular dichroism to show that aSyn with acK at position 43 has less alpha-helical content. From this result, they deduce that "only this site could potentially perturb aS function in neurotransmitter trafficking", but no experiments on neurotransmitter trafficking were performed.
We agree with the reviewer that neurotransmitter trafficking studies would be interesting, but they would presumably require the use of acetylation mimic mutants (Lys-to-Gln mutations), which we would want to validate by comparison to our semi-synthetic proteins with authentic AcK. Such experiments are planned for a follow-up manuscript, and we will investigate the reviewer’s suggested experiment at …
Author response:
The following is the authors’ response to the original reviews.
Public Reviews:
Reviewer #1 (Public review):
Weaknesses:
The authors then use circular dichroism to show that aSyn with acK at position 43 has less alpha-helical content. From this result, they deduce that "only this site could potentially perturb aS function in neurotransmitter trafficking", but no experiments on neurotransmitter trafficking were performed.
We agree with the reviewer that neurotransmitter trafficking studies would be interesting, but they would presumably require the use of acetylation mimic mutants (Lys-to-Gln mutations), which we would want to validate by comparison to our semi-synthetic proteins with authentic AcK. Such experiments are planned for a follow-up manuscript, and we will investigate the reviewer’s suggested experiment at that time. Thus, we have not modified the manuscript to address this issue.
Subsequently, they measure the aggregation speed of the variants in seeded aggregation experiments with preformed fibrils (PFFs) from WT aSyn, and conclude that acK at positions 12, 43, and 80 yields slower aggregation. They reach similar conclusions when measuring seeded aggregation in primary cultures. As far as I understand it, the seeding experiments in cells use seeds that are assembled from partially acetylated alpha-synuclein, but that are made of non-acetylated wildtype alpha-synuclein, and the alpha-synuclein that is endogenous in the cells is also non-acetylated (or at least not beyond what happens in these cells at endogenous levels). It is therefore unclear how the cellular seeding experiments relate to the in vitro aggregation assays with (partially) acetylated substrates.
We understand the reviewer’s concerns and have modified the manuscript to clarify that the method of in vitro seeding really reports on the impact of acetylation on the elongation phase of aggregation. We have also clarified that this is different than the role that acetylation plays in seeding cellular aggregation with pre-acetylated fibrils. We note that having the monomer population acetylated in cells presents technical challenges that might also be addressed with Gln mutant mimics, and we plan to pursue such experiments in the follow-up manuscript described above.
Anyway, both aggregation experiments ignore that the structures of aSyn filaments in Parkinson's disease (PD) or multiple system atrophy (MSA) are different from those formed in these experiments, and that, therefore, the observed aggregation kinetics are likely irrelevant for the speed with which disease-relevant filaments form in the brain.
Finally, the authors describe the cryo-EM structure of mixtures of acK80:WT aSyn filaments, which are predominantly made of WT aSyn, with a previously described structure. Filaments made of only acK80 aSyn have a modified arrangement of this structure, where the now neutral side chain of residue 80 packs inside a hydrophobic pocket. The authors discuss differences between the acK80 structures and those of other structures from in vitro assembled aSyn filaments, none of which are the same as those observed from PD or MSA brains, nor are any attempts made to transfer observations from the in vitro experiments to the structures of disease. The relevance of the cryo-EM structures for human disease, therefore, remains unclear.
The Conclusion on p.20 mentions an interesting and valuable result: the authors used the acetylated recombinant proteins to determine the extent of acetylation within human protein samples by quantitative liquid chromatography MS (SI, Figures S41-S49). Their conclusion is that "The level of acetylation was variable - no clear trend was observed between healthy control and patients - nor between patients of different diseases (SI, Table S4, Supplementary Data 1)" This result implies that acetylation of aS is not directly related to its pathogenicity, which again adds doubts on the disease-relevance of the results described in the rest of the paper.
We acknowledge the concerns raised in the above paragraphs and believe that they can all be addressed by clarifying our purpose. The different fibril polymorphs adopted in PD and MSA are likely the result of an interplay of many PTMs and non-proteinaceous cofactors. Therefore, we are not necessarily trying to claim that our AcK80 fold is populated in health or disease, but that by driving Lys80 acetylation, one could push fibrils to adopt this conformation, which is less aggregation-prone. A similar argument has been made in investigations of alpha-synuclein glycosylation and phosphorylation. Our results in Figure 9 imply that Lys80 acetylation could be increased with HDAC8 inhibition. We have revised the manuscript to make these ideas clearer, while being sure to acknowledge the limitations noted by Reviewer #1.
Reviewer #2 (Public review):
Weaknesses:
SDS is not a good membrane model to investigate the effect of lysine acetylation on aS membrane binding because it is a harsh detergent and solubilizes membranes. Negatively charged vesicles or vesicles made of a mixture of lipids mimicking the lipid composition of synaptic vesicles are more accepted in the field to study aS-membrane interactions. The authors used such vesicles for the FCS experiments, and they could be used for the initial screening of the 12 lysine acetylated variants of aS.
We have noted this shortcoming in revisions of our manuscript, but have not performed new experiments as we do not believe that using vesicles instead would change the conclusions of these experiments (that only AcK43 produces an effect, and a modest one at that).
It would help the reader to have the experimental details (e.g., buffer, protein/lipid concentrations) for the different assays written in the figure legend.
We have added additional detail to the figure captions.
The authors use an assay consisting of mixing 10% fibrils + 90% monomer to investigate the effect of lysine acetylation on aS. However, the assay only probes fibril elongation and/or secondary processes. The current wording can be misleading, and the term aggregation could be replaced by seeding capacity for clarity. For example, the authors state that lysine acetylation at sites 12, 43, and 80 each inhibits aggregation, but this statement is not supported by the data. Instead, the data show that the acetylation at these sites slows down the fibril elongation and thus decreases the seeding capacity of aS fibrils. In order to state that lysine acetylation has an effect on aS aggregation, fibril formation, the author should use an assay where the de novo formation of fibrils is assessed, such as in the presence of lipid vesicles or under shaking conditions.
As noted in our response to Reviewer #1, we have clarified which phase of aggregation we were investigating in our in vitro experiments.
It is not clear from the EM data that the structures of the different lysine acetylated variants are different, unlike what is stated in the text.
We feel that it is clear from structures in Figure 8 and the EM density maps in Figure S38 that the AcK80 fold is indeed different. Although the overall polymorphs are somewhat similar to WT, the position of K80 clearly changes upon acetylation, altering the local fold significantly and the global fold more moderately. We have added backbone RMSD calculations to quantify the differences in WT and AcK80 folds in Figure SX. They differ by ~5 Å in the fibril core region.
Reviewer #3 (Public review):
Weaknesses:
The challenges the authors report regarding semi-synthetic access to aSyn are somewhat surprising, as this protein has been made by a variety of different semi-synthesis strategies in satisfactory yields and without similar problems being reported.
We understand the reviewer’s surprise and have edited the manuscript to clarify that the NCL yields were not unusually low, but were comparable to ncAA yields, and since it is significantly easier to scan AcK positions using ncAAs, we felt that ncAAs are the method of choice in this case.
Recommendations for the authors:
Reviewer #1 (Recommendations for the authors):
(1) Cryo-EM data processing: particles were pre-processed in cryosparc and ChatGPT-generated scripts. Are priors on tilt and psi angles defined through this procedure? And are segments from individual filaments kept strictly in the same half-sets for gold-standard estimation of resolution? Absence of psi and tilt priors will lead to worse refinements than otherwise possible. Worse, a mixture of segments from different filaments into the two half-sets may lead to overestimated resolution estimates.
We thank the reviewer for their thoughtful analysis of our cryo-EM data processing approach. In response, we have modified our approach and added additional commentary on processing to the Materials and Methods section.
“CryoSPARC (.cs) files were then converted to RELION STAR files using the PyEM csparc2star.py script. Following this data conversion, a custom Python script developed with ChatGPT precisely determined the start and end coordinates of each fibril. This script processed the csparc2star.py star file output to create coordinate pairs based on the cryoSPARC Fibril ID, notably without transferring the original tilt and psi angles from CryoSPARC to RELION. The output of this custom script served as the input for the autopick RELION extraction step.
To handle curved fibrils, a special segmentation strategy was implemented: the script traced the coordinates along the fibril, generating a new start and end coordinate pair for individal segments, with the segment's end coordinate assigned either after spanning 10 particles (around 50 nm in length) or when the end of the fibril was reached. This resulted in shorter, straighter segments for processing. Finally, the createAutopick function from cryolo_boxmanager_tools.py in crYOLO was utilized to generate a STAR file linking the final particle coordinates to their movie files, which was then used to perform particle extraction in RELION. The standard RELION image processing pipeline then followed, including 2D classification, refinement, and 3D classification.
This approach resolves the issue with curved fibrils, but also results in all picked fibrils being 50 nm or shorter in RELION. Consequently, segments from the same fibril receive unique fibril IDs in RELION and may be split into different half-maps. Although this avoids random splitting of individual particles without regard to their origin from the same fibril, it could still cause an overestimation of resolution.
To assess any potential overestimation of resolution, another script was created to reassign the fibril ID of each particle in the RELION STAR file to that of the closest particles in the cryoSPRAC data, effectively ensuring that all particles from an individual fibril have the same fibril ID and are not assigned to different half-maps. This revised STAR file was then used as the input images STAR file for 3D auto-refinement in RELION. A comparison of maps before and after reassigning the fibril IDs shows negligible effects on the resulting structures and on their estimated resolution, indicating that the original procedure did not results in any significant overestimation of the resolution.”
Author response image 1.
RELION Cryo-EM maps before (gray) and after (yellow) fibril ID reassignment for (A) WT-A (B) WT-B (C) AcK80-A (D) AcK80-B, showing that the new processing approaches did not significantly change the fibril structures.
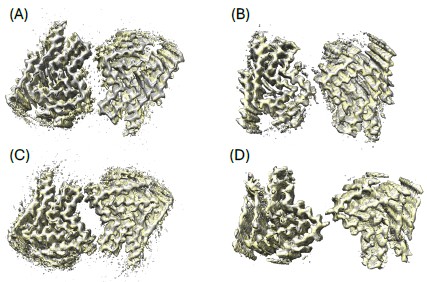
(2) The 25% acK80 structure in S52 is understood to be wildtype-only. The authors mention in the main text that this is because of the strong density for the K80 side chain. An additional argument would be that an acK80 would leave an unshielded negative charge on the neighbouring E46, as K80 and E46 form a salt bridge in this structure.
We appreciate the reviewer’s idea and have included a comment on the salt bridge impact.
(3) It would be valuable to include side views of the density for all reported reconstructions to assess to what extent the beta-rungs are separated.
The requested side views have been included in Figure SX.
(4) Methods sections should be moved into the main text of the paper.
This Materials and Methods portion of Supporting Information has been moved to the main text.
Reviewer #3 (Recommendations for the authors):
(1) We suggest removing "all" from the manuscript title as this claim might not hold up in the future.
We understand the reviewer’s concern. Our title was meant to imply “all currently known” rather than “all” forever, but as this wording is awkward, we have deleted “all” as suggested.
(2) The white font in Figure 1A is sometimes hard to read, especially on the yellow-green background between amino acids 70-80.
We have changed this to black font.
Figure 1 panels C-E are not referenced in the manuscript text?
References to the Figure 1 panels have been added.
In panel C, a structure is predicted, but based on what data? Why is there both a small and a big structure in panel C?
Explanations of the Figure 1C images have been added to the caption.
(3) Typo ε-acetyllysine -> Nε-acetyllysine
This has been corrected throughout.
(4) You report solubility issues during NCL, and these are typically alleviated by the use of chaotropes during ligation. Please specify what you mean by "standard NCL conditions" and include parameters such as guanidine concentration, pH, concentrations, volumes, and temperature.
These details have now been added to the methods section.
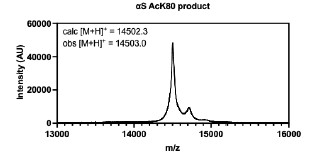
(5) According to Figure 2D, the desulfurization was incomplete. Please explain.
The small peak observed next to the product peak is an adduct with sinapic acid (+206 Da), the matrix mixed in for MALDI acquisition. We do not see a sign of +32/64Da peak which would correspond to incomplete desulfurization
Author response image 2.
(6) Please include sequences of your constructs for ncAA mutagenesis. Especially, which intein was attached at what position. This is important for other groups to fully understand the production of acetylated aSyn variants.
The full DNA sequence has been added to Supporting Information. This plasmid has also been reported previously in the referenced publications.
(7) You state ncAA mutagenesis "yielded 0.11-1.5 mg" aSyn. I guess this is per-liter culture expression medium?
This has been corrected.
(8) The resolution/DPI of Figures 4, 5, S14-16, and S18 should be increased. They look blurred compared to Figures 6 or S19.
These figures have been updated.
(9) You provided only summaries in Figures 4 and 5 because of space restrictions. However, it would be nice to have at least some selected individual experiments (WT, acetylation K12/43/80) right next to it without the need to switch to S14, S15, or S16.
Select experimental data has been added to main text Figures 4 and 5 as requested.
(10) Please increase the size of the microscopy images in Figure 6 (in Figure S19, it looks much better).
This size of the images in Figure 6 has been increased.
(11) The labelling A1-A3 in Figure S33 was somehow unclear to me.
These three panels show different sections of the TEM grid, illustrating heterogeneity in the 25% AcK12 fibrils that was not observed for fibrils of the other acetylation variants. We have clarified this in the figure caption.
(12) In Figure 9, you present preliminary results regarding site-specific deacetylation by HDAC8. These results are interesting, but considering the exploratory nature of this in vitro experiment, I suggest toning down the highly enthusiastic discussion of potential in vivo effects.
We understand the reviewer’s concern and have mitigated the claims of potential impact from these in vitro results.
-

-
-

-
-
-
eLife Assessment
This valuable work provides new insights into the role of lysine acetylation of alpha-synuclein, the protein involved in Parkinson's Disease. The evidence is mostly solid, but the claims around the potential disease relevance based on seeding assays and structural work need to be toned down, or else supported by additional experimental evidence. Overall, the work will be of interest to researchers in the fields of protein biophysics and post-translational modifications, as well as Parkinson's Disease.
-
Reviewer #1 (Public review):
Summary:
This paper describes experiments with alpha-synuclein (aS) with acetylated lysines (acK) at various positions. Their findings on how to use non-canonical amino acid (ncAA) mutagenesis to generate aS with acetylated lysines are valuable. The paper then continues with a range of experiments to characterise the acetylated alpha-synuclein constructs at different positions, with the aim of providing insights into which sites are relevant to disease or their function inside cells. The paper concludes these experiments with the suggestion that inhibiting the Zn2+-dependent histone deacetylase HDAC8 to potentially increase acetylation at lysine 80 may have therapeutic benefit. However, the relevance of most of these experiments is unclear, mainly as the filaments that form from these constructs are …
Reviewer #1 (Public review):
Summary:
This paper describes experiments with alpha-synuclein (aS) with acetylated lysines (acK) at various positions. Their findings on how to use non-canonical amino acid (ncAA) mutagenesis to generate aS with acetylated lysines are valuable. The paper then continues with a range of experiments to characterise the acetylated alpha-synuclein constructs at different positions, with the aim of providing insights into which sites are relevant to disease or their function inside cells. The paper concludes these experiments with the suggestion that inhibiting the Zn2+-dependent histone deacetylase HDAC8 to potentially increase acetylation at lysine 80 may have therapeutic benefit. However, the relevance of most of these experiments is unclear, mainly as the filaments that form from these constructs are different from those observed in human disease (but see below for more details). Moreover, using the recombinantly produced acetylated versions of alpha-synuclein to normalise mass-spectrometry data, the authors themselves report that acetylation of alpha-synuclein does not differ between individuals with Parkinson's disease or healthy controls.
Strengths:
The authors report difficulties with chemical synthesis, and then decide to make these constructs using non-canonical amino acid (ncAA) mutagenesis, which seems to work reasonably well (yields vary somewhat). In the Conclusion section, the authors report that they used these recombinant proteins to obtain quantitative insights into the levels of acetylation of lysines in individuals with PD versus healthy controls, for which they find no significant differences. This part of the work is valuable.
Weaknesses:
The authors then use circular dichroism to show that aSyn with acK at position 43 has less alpha-helical content. From this result, they deduce that "only this site could potentially perturb aS function in neurotransmitter trafficking", but no experiments on neurotransmitter trafficking were performed.
Subsequently, they measure the aggregation speed of the variants in seeded aggregation experiments with preformed fibrils (PFFs) from WT aSyn, and conclude that acK at positions 12, 43, and 80 yields slower aggregation. They reach similar conclusions when measuring seeded aggregation in primary cultures. As far as I understand it, the seeding experiments in cells use seeds that are assembled from partially acetylated alpha-synuclein, but that are made of non-acetylated wildtype alpha-synuclein, and the alpha-synuclein that is endogenous in the cells is also non-acetylated (or at least not beyond what happens in these cells at endogenous levels). It is therefore unclear how the cellular seeding experiments relate to the in vitro aggregation assays with (partially) acetylated substrates. Anyway, both aggregation experiments ignore that the structures of aSyn filaments in Parkinson's disease (PD) or multiple system atrophy (MSA) are different from those formed in these experiments, and that, therefore, the observed aggregation kinetics are likely irrelevant for the speed with which disease-relevant filaments form in the brain.
NMR and FCS experiments show that acK at positions 12 and 43 may reduce binding to vesicles, which then leaves only acK80.
Finally, the authors describe the cryo-EM structure of mixtures of acK80:WT aSyn filaments, which are predominantly made of WT aSyn, with a previously described structure. Filaments made of only acK80 aSyn have a modified arrangement of this structure, where the now neutral side chain of residue 80 packs inside a hydrophobic pocket. The authors discuss differences between the acK80 structures and those of other structures from in vitro assembled aSyn filaments, none of which are the same as those observed from PD or MSA brains, nor are any attempts made to transfer observations from the in vitro experiments to the structures of disease. The relevance of the cryo-EM structures for human disease, therefore, remains unclear.
The Conclusion on p.20 mentions an interesting and valuable result: the authors used the acetylated recombinant proteins to determine the extent of acetylation within human protein samples by quantitative liquid chromatography MS (SI, Figures S41-S49). Their conclusion is that "The level of acetylation was variable - no clear trend was observed between healthy control and patients - nor between patients of different diseases (SI, Table S4, Supplementary Data 1)" This result implies that acetylation of aS is not directly related to its pathogenicity, which again adds doubts on the disease-relevance of the results described in the rest of the paper.
-
Reviewer #2 (Public review):
Summary:
Shimogawa et al. studied the effect of lysine acetylation at different sites in the alpha-synuclein (aS) sequence on the protein-membrane affinity, seeding capacity in the test tube and in cells, and on the structure of fibrils, using a range of biophysical methods. They use non-canonical amino acid (ncAA) mutagenesis to prepare aS lysine acetylated variant at different sites.
Strengths:
The major strength of this paper is the approach used for the production of site-specific lysine acetylated variants of aS using ncAA mutagenesis, as well as the combination of a range of biophysical methods together with cellular assays and structure biology to decipher the effect of lysine acetylation on aS-membrane binding, seeding propensity, and fibril structure. This approach allowed the author to find that …
Reviewer #2 (Public review):
Summary:
Shimogawa et al. studied the effect of lysine acetylation at different sites in the alpha-synuclein (aS) sequence on the protein-membrane affinity, seeding capacity in the test tube and in cells, and on the structure of fibrils, using a range of biophysical methods. They use non-canonical amino acid (ncAA) mutagenesis to prepare aS lysine acetylated variant at different sites.
Strengths:
The major strength of this paper is the approach used for the production of site-specific lysine acetylated variants of aS using ncAA mutagenesis, as well as the combination of a range of biophysical methods together with cellular assays and structure biology to decipher the effect of lysine acetylation on aS-membrane binding, seeding propensity, and fibril structure. This approach allowed the author to find that lysine acetylation at positions 12, 43, and 80 led to lower seeding capacity of aS in the test tube and in cells, but only acetylation at lysine 80 did not affect aS-membrane interaction. These results suggest that lysine acetylation at position 80 may be protective against aggregation without perturbing the proposed functional role of aS in synaptic plasticity.
Weaknesses:
SDS is not a good membrane model to investigate the effect of lysine acetylation on aS membrane-binding because it is a harsh detergent and solubilizes membranes. Negatively charged vesicles or vesicles made of a mixture of lipids mimicking the lipid composition of synaptic vesicles are more accepted in the field to study aS-membrane interactions. The authors used such vesicles for the FCS experiments, and they could be used for the initial screening of the 12 lysine acetylated variants of aS.
It would help the reader to have the experimental details (e.g., buffer, protein/lipid concentrations) for the different assays written in the figure legend.
The authors use an assay consisting of mixing 10% fibrils + 90% monomer to investigate the effect of lysine acetylation on aS. However, the assay only probes fibril elongation and/or secondary processes. The current wording can be misleading, and the term aggregation could be replaced by seeding capacity for clarity. For example, the authors state that lysine acetylation at sites 12, 43, and 80 each inhibits aggregation, but this statement is not supported by the data. Instead, the data show that the acetylation at these sites slows down the fibril elongation and thus decreases the seeding capacity of aS fibrils. In order to state that lysine acetylation has an effect on aS aggregation, fibril formation, the author should use an assay where the de novo formation of fibrils is assessed, such as in the presence of lipid vesicles or under shaking conditions.
It is not clear from the EM data that the structures of the different lysine acetylated variants are different, unlike what is stated in the text.
-
Reviewer #3 (Public review):
Shimogawa et al. describe the generation of acetylated aSyn variants by genetic code expansion to elucidate effects on vesicle binding, aggregation, and seeding effects. The authors compared a semi-synthetic approach to obtain acetylated aSyn variants with genetic code expansion and concluded that the latter was more efficient in generating all 12 variants studied here, despite the low yields for some of them. Selected acetylated variants were used in advanced NMR, FCS, and cryo-EM experiments to elucidate structural and functional changes caused by acetylation of aSyn. Finally, site-specific differences in deacetylation by HDAC 8 were identified.
The study is of high scientific quality, andthe results are convincingly supported by the experimental data provided. The challenges the authors report regarding …
Reviewer #3 (Public review):
Shimogawa et al. describe the generation of acetylated aSyn variants by genetic code expansion to elucidate effects on vesicle binding, aggregation, and seeding effects. The authors compared a semi-synthetic approach to obtain acetylated aSyn variants with genetic code expansion and concluded that the latter was more efficient in generating all 12 variants studied here, despite the low yields for some of them. Selected acetylated variants were used in advanced NMR, FCS, and cryo-EM experiments to elucidate structural and functional changes caused by acetylation of aSyn. Finally, site-specific differences in deacetylation by HDAC 8 were identified.
The study is of high scientific quality, andthe results are convincingly supported by the experimental data provided. The challenges the authors report regarding semi-synthetic access to aSyn are somewhat surprising, as this protein has been made by a variety of different semi-synthesis strategies in satisfactory yields and without similar problems being reported.
The role of PTMs such as acetylation in neurodegenerative diseases is of high relevance for the field, and a particular strength of this study is the use of authentic acetylated aSyn instead of acetylation-mimicking mutations. The finding that certain lysine acetylations can slow down aggregation even when present only at 10-25% of total aSyn is exciting and bears some potential for diagnostics and therapeutic intervention.
-
Author response:
We thank you for your efforts in reviewing our manuscript. We sincerely appreciate that the reviewers were all enthusiastic about our comparison of native chemical ligation (NCL) and non-canonical amino acid (ncAA) mutagenesis methods for installing acetyl lysine (AcK) in alpha-synuclein, as well as the wide variety of biochemical experiments enabled by our ncAA approach. We respond to the critiques specific to each reviewer here.
Reviewer #1:
Expressed concern that in vitro studies of effects on membrane binding were not followed up with neurotransmitter trafficking experiments. While we certainly think that such studies would be interesting, they would presumably require the use of acetylation mimic mutants (Lys-to-Gln mutations), which we would want to validate by comparison to our semi-synthetic proteins with …
Author response:
We thank you for your efforts in reviewing our manuscript. We sincerely appreciate that the reviewers were all enthusiastic about our comparison of native chemical ligation (NCL) and non-canonical amino acid (ncAA) mutagenesis methods for installing acetyl lysine (AcK) in alpha-synuclein, as well as the wide variety of biochemical experiments enabled by our ncAA approach. We respond to the critiques specific to each reviewer here.
Reviewer #1:
Expressed concern that in vitro studies of effects on membrane binding were not followed up with neurotransmitter trafficking experiments. While we certainly think that such studies would be interesting, they would presumably require the use of acetylation mimic mutants (Lys-to-Gln mutations), which we would want to validate by comparison to our semi-synthetic proteins with authentic AcK. Such experiments are planned for a follow-up manuscript, and we will investigate the reviewer’s suggested experiment at that time.
Reviewer #1 Noted that the method of in vitro seeding really reports on the impact of acetylation on the elongation phase of aggregation. We will clarify this in our revisions. They also expressed concern that this was different than the role that acetylation would play in seeding cellular aggregation with pre-acetylated fibrils. We will also acknowledge and clarify this in our revisions. Having the monomer population acetylated in cells presents technical challenges that might also be addressed with Gln mutant mimics, and we plan to pursue such experiments in the follow-up manuscript noted above.
Reviewer #1 Criticized the fact that the pre-formed fibrils used in seeding would not have the same polymorph as PD or MSA fibrils derived from patient material. They were also critical of how our cryo-EM structure of AcK80 fibrils related to the PD and MSA polymorphs. Finally, while the reviewer liked the MS experiments used to quantify acetylation levels from patient samples, they felt that our findings then threw the physiological relevance of our structural and biochemical experiments into question. We believe that all of these critiques can be addressed by clarifying our purpose. We are not necessarily trying to claim that our AcK80 fold is populated in health or disease, but that by driving Lys80 acetylation, one could push fibrils to adopt this conformation, which is less aggregation-prone. A similar argument has been made in investigations of alpha-synuclein glycosylation and phosphorylation. Our results in Figure 9 imply that this could be done with HDAC8 inhibition. We will revise the manuscript to make these ideas clearer, while being sure to acknowledge the limitations noted by Reviewer #1.
Reviewer #2:
Expressed concern over our use of SDS micelles for initial investigation of the 12 AcK variants, rather than the phospholipid vesicles used in later FCS and NMR experiments. We will note this shortcoming in revisions of our manuscript, but we do not believe that using vesicles instead would change the conclusions of these experiments (that only AcK43 produces an effect, and a modest one at that).
We will add additional detail to the figure captions, as requested by Reviewer #2.
Reviewer #2 shared some of the concerns of Reviewer #1 regarding the distinctions of which phase of aggregation we were investigating in our in vitro experiments. As noted above, we will clarify this language.
Finally, Reviewer #2 stated that “It is not clear from the EM data that the structures of the different lysine acetylated variants are different.” We feel that it is quite clear from structures in Figure 8 and the EM density maps in Figure S38 that the AcK80 fold is indeed different. Although the overall polymorphs are somewhat similar to WT, the position of K80 clearly changes upon acetylation, altering the local fold significantly and the global fold more moderately.
Reviewer #3:
Found the results convincing, including the potential therapeutic implications. The only concern noted was that they found the difficulties in semi-synthesis of AcK-modified alpha-synuclein surprising given that it has been made many times before through NCL. Indeed, our own laboratory has made alpha-synuclein through NCL, and the yields reported here are in keeping with our own previous results. However, since NCL did not give higher yields than ncAA methods, and it is significantly easier to scan AcK positions using ncAAs, we felt that ncAAs are the method of choice in this case. We will clarify this position in the revised manuscript.
In conclusion, on behalf of all authors, I again thank the reviewers for both their positive and negative observations in helping us to improve our manuscript. We will revise it to strive for greater clarity as we have noted in this letter.
-
-
-