Adaptive behavior is guided by integrated representations of controlled and non-controlled information
Curation statements for this article:-
Curated by eLife

eLife Assessment
This useful study uses creative scalp EEG decoding methods to attempt to demonstrate that two forms of learned associations in a Stroop task are dissociable, despite sharing similar temporal dynamics. However, the evidence supporting the conclusions is incomplete due to concerns with the experimental design and methodology. This paper would be of interest to researchers studying cognitive control and adaptive behavior, if the concerns raised in the reviews can be addressed satisfactorily.
This article has been Reviewed by the following groups
Listed in
- Evaluated articles (eLife)
Abstract
Understanding how task knowledge is encoded neurally is crucial for uncovering the mechanisms underlying adaptive behavior. Here, we test the theory that all task information is integrated into a conjunctive task representation by investigating whether this representation simultaneously includes two types of associations that can guide behavior: stimulus–response (non-controlled) associations and stimulus–control (controlled) associations that inform how task focus should be adjusted to achieve goal-directed behavior. We extended the classic item-specific proportion congruency paradigm to dissociate the electroencephalographic (EEG) representations of controlled and non-controlled associations. Behavioral data replicated previous findings of association-driven adaptive behaviors. Decoding analyses of EEG data further showed that associations of controlled and non-controlled information were represented concurrently and differentially. Brain-behavioral analyses also showed that the strength of both associations was associated with faster responses. These findings provide initial evidence supporting the idea that controlled and non-controlled associations are governed by an integrated task representation to guide adaptive behaviors simultaneously.
Article activity feed
-
Adaptive behavior is guided by integrated representations of controlled and non-controlled information elifesciences.org/articles/108...
-

-
-
-
-

eLife Assessment
This useful study uses creative scalp EEG decoding methods to attempt to demonstrate that two forms of learned associations in a Stroop task are dissociable, despite sharing similar temporal dynamics. However, the evidence supporting the conclusions is incomplete due to concerns with the experimental design and methodology. This paper would be of interest to researchers studying cognitive control and adaptive behavior, if the concerns raised in the reviews can be addressed satisfactorily.
-
Reviewer #1 (Public review):
Summary:
This study focuses on characterizing the EEG correlates of item-specific proportion congruency effects. In particular, two types of learned associations are studied. One association involves associations between stimulus features and control states (SC), and the other involves stimulus features and responses (SR). Decoding methods are used to identify time-resolved SC and SR correlates.
The authors conclude that SC and SR associations can independently and simultaneously guide behavior. This conclusion is based on results showing that SC and SR correlates are (1) not entirely overlapping in cross-decoding, (2) simultaneously observed on average over trials, (3) independently correlate with RT, and (4) have a positive within-trial correlation.
Strengths:
Fearless, creative use of EEG decoding to test …
Reviewer #1 (Public review):
Summary:
This study focuses on characterizing the EEG correlates of item-specific proportion congruency effects. In particular, two types of learned associations are studied. One association involves associations between stimulus features and control states (SC), and the other involves stimulus features and responses (SR). Decoding methods are used to identify time-resolved SC and SR correlates.
The authors conclude that SC and SR associations can independently and simultaneously guide behavior. This conclusion is based on results showing that SC and SR correlates are (1) not entirely overlapping in cross-decoding, (2) simultaneously observed on average over trials, (3) independently correlate with RT, and (4) have a positive within-trial correlation.
Strengths:
Fearless, creative use of EEG decoding to test tricky hypotheses regarding latent associations.
Nice idea to orthogonalize ISPC condition (MC/MI) from stimulus features.
Response:
In their last response to the reviewers, the authors write:
"... constructing a theoretically unbiased decoder requires perfectly counter-balanced training data (i.e., for every training trial of class A that is X trials away from the test data, there must be a training trial of all other classes that is exactly X trials away from the test data). As we were unable to achieve such a perfect design, we chose not to run an additional experiment."
This isn't really an issue about whether this design is "perfectly" orthogonal. It's an issue regarding a clear confound among the decoded classes for SC/SR decoders. To be clear: of the 8 classes in the SC decoder, 4 are overwhelmingly presented in the first half (PHASE 2) of the session, whereas the other 4 are overwhelmingly presented in the second half (PHASE 3). The same is true for the SR decoder. So, session-half correlated noise could readily contribute to distinguishing among these classes. And counterbalancing this across subjects won't help because decoders lose sign.
To me, the conducted control analyses don't really make strong contact with this issue. The split-half cross-validation is a nice idea but, as the authors acknowledge, it's also subject to slower cross-session noise, as is the original analysis. This sort of noise is not exactly exotic in EEG. Caps/hair/electrodes shift, gel dries and impedance changes, posture / muscle tension / skin conductance changes, fatigue may wax and wane (e.g., linked to increasing alpha), etc. And the newest analysis didn't really seem to engage with this issue either, as it only assessed minimum distances between classes, on the order of 5 +- 2 SD trials. This seems to assume that the dominant potential sources of noise will be scale-free, such that the strength of the relation at short time scales would generalize to longer ones. I'm not sure why that's expected here.
Here are some suggestions for alternative control analyses that I think would be more targeted to this issue:
(1) Explicitly train a decoder to separate the three levels of PHASE from each other. Successful decoding would provide positive evidence for the presence of structured noise at this timescale.
(2) Specify an RDM for the PHASE variable and regress this component separately from each time-point/trial of the SC and SR decoders. This is a post-hoc band-aid, but it is in the spirit of correcting for a known confound.
(3) In the spirit of the authors' distance analysis, but without assuming that the noise is scale-free: perform a time-series RSA like that in Alink et al. (2015; https://doi.org/10.1101/032391), Fig. 1 and 3. This would allow one, e.g., to estimate the structure & timescales of the noise processes across the session.
Other readers may, like me, be puzzled by the selection of this particular experimental design to test this question of SC and SR coding, given the temporal confound among SC/SR classes, and given that there would seem to be many possible designs that are less confounded. For example, why not use a design where ISPC was swapped/shuffled several more times within each subject, so that PHASE is more orthogonal to long-timescale noise? Isn't ISPC learning fast enough to support learning phases shorter than 700 trials? Such readers would likely appreciate a frank discussion of this dilemma, and a motivation for the choice of the present design, within the manuscript.
Pre-stimulus coding:
To explain the apparent pre-stimulus coding of several task variables, the newest version of the manuscript proposes that subjects were proactively coding these variables via predictive mechanisms. This is an interesting account of item-specific control. It is also surprising, given that item-specific control mechanisms are typically conceptualized as reactive or stimulus-driven phenomena. But I think support for a proactive control account was incomplete. The mechanistic logic was not presented, and no hypotheses under this account were developed or tested. So I would suggest pinning down some hypotheses here and actually putting this account to the test.
Outliers & t-values: thank you for checking this!
Random slopes were omitted due to convergence failure, but this can inflate false positive inferences (e.g., Barr et al. 2013), and doesn't really motivate a minimal model. I'd suggest trying a slightly reduced model (e.g., drop correlations via `slope || subject`) using buildMer automated selection, or switching to brms.
-
Reviewer #2 (Public review):
Summary:
In this EEG study, Huang et al. investigated the relative contribution of two accounts to the process of conflict control, namely the stimulus-control association (SC), which refers to the phenomenon that the ratio of congruent vs. incongruent trials affects the overall control demands, and the stimulus-response association (SR), stating that the frequency of stimulus-response pairings can also impact the level of control. The authors extended the Stroop task with novel manipulation of item congruencies across blocks in order to test whether both types of information are encoded and related to behaviour. Using decoding and RSA they showed that the SC and SR representations were concurrently present in voltage signals and they also positively co-varied. In addition, the variability in both of their …
Reviewer #2 (Public review):
Summary:
In this EEG study, Huang et al. investigated the relative contribution of two accounts to the process of conflict control, namely the stimulus-control association (SC), which refers to the phenomenon that the ratio of congruent vs. incongruent trials affects the overall control demands, and the stimulus-response association (SR), stating that the frequency of stimulus-response pairings can also impact the level of control. The authors extended the Stroop task with novel manipulation of item congruencies across blocks in order to test whether both types of information are encoded and related to behaviour. Using decoding and RSA they showed that the SC and SR representations were concurrently present in voltage signals and they also positively co-varied. In addition, the variability in both of their strengths was predictive of reaction time. In general, the experiment has a solid design and the analyses are appropriate for the research questions.
Strengths:
(1) The authors used an interesting task design that extended the classic Stroop paradigm and is effective in teasing apart the relative contribution of the two different accounts regarding item-specific proportion congruency effect.
(2) Linking the strength of RSA scores with behavioural measure is critical to demonstrating the functional significance of the task representations in question.
Weaknesses:
I still have some doubts on the effectiveness of the experimental manipulation on Phase 2: although the ISPC effect is still present, it is much weaker in comparison, suggesting the participants did not learn the contingency statistics in Phase 2 as well as they did in the other phases, due to either the lingering effect of the previous phase or an inherent bias towards one color pairs. Perhaps by separately plotting the earlier and later blocks of Phase 2 any difference can be revealed if it exists. This behavioral difference could result in unequal levels of SC/SR representation across phases, which may raise problems when data were combined for analyses that assume the neural effects are equivalent.
-
Author response:
The following is the authors’ response to the previous reviews
eLife Assessment
This useful study uses creative scalp EEG decoding methods to attempt to demonstrate that two forms of learned associations in a Stroop task are dissociable, despite sharing similar temporal dynamics. However, the evidence supporting the conclusions is incomplete due to concerns with the experimental design and methodology. This paper would be of interest to researchers studying cognitive control and adaptive behavior, if the concerns raised in the reviews can be addressed satisfactorily.
We thank the editors and the reviewers for their positive assessment and constructive feedback of our work, which led us to think more deeply about the conceptual and methodological aspects of this project and further strengthen the manuscript. Based on …
Author response:
The following is the authors’ response to the previous reviews
eLife Assessment
This useful study uses creative scalp EEG decoding methods to attempt to demonstrate that two forms of learned associations in a Stroop task are dissociable, despite sharing similar temporal dynamics. However, the evidence supporting the conclusions is incomplete due to concerns with the experimental design and methodology. This paper would be of interest to researchers studying cognitive control and adaptive behavior, if the concerns raised in the reviews can be addressed satisfactorily.
We thank the editors and the reviewers for their positive assessment and constructive feedback of our work, which led us to think more deeply about the conceptual and methodological aspects of this project and further strengthen the manuscript. Based on the comments, we included more control analyses and revised the manuscript accordingly. Please see below our responses to each comment raised in the reviews.
Public Reviews:
Reviewer #1 (Public review):
Summary:
This study focuses on characterizing the EEG correlates of item-specific proportion congruency effects. Two types of learned associations are characterized, one being associations between stimulus features and control states (SC), and the other being stimulus features and responses (SR). Decoding methods are used to identify time-resolved SC and SR correlates, which are used to test properties of their dynamics.
The conclusion is reached that SC and SR associations can independently and simultaneously guide behavior. This conclusion is based on results showing SC and SR correlates are: (1) not entirely overlapping in cross-decoding; (2) simultaneously observed on average over trials in overlapping time bins; (3) independently correlate with RT; and (4) have a positive within-trial correlation.
Strengths:
Fearless, creative use of EEG decoding to test tricky hypotheses regarding latent associations.
Nice idea to orthogonalize ISPC condition (MC/MI) from stimulus features.
Thank you for acknowledging the strength in EEG decoding and design. We have addressed all your concerns raised below point by point.
Weaknesses:
I still have my concern from the first round that the decoders are overfit to temporally structured noise. As I wrote before, the SC and SR classes are highly confounded with phase (chunk of session). I do not see how the control analyses conducted in the revision adequately deal with this issue.
In the figures, there are several hints that these decoders are biased. Unfortunately, the figures are also constructed in such a way that hides or diminishes the salience of the clues of bias. This bias and lack of transparency discourage trust in the methods and results.
I have two main suggestions:
(1) Run a new experiment with a design that properly supports this question.
I don't make this suggestion lightly, and I understand that it may not be feasible to implement given constraints; but I feel that this suggestion is warranted. The desired inferences rely on successful identification of SC and SR representations. Solidly identifying SC and SR representations necessitates an experimental design wherein these variables are sufficiently orthogonalized, within-subject, from temporally structured noise. The experimental design reported in this paper unfortunately does not meet this bar, in my opinion (and the opinion of a colleague I solicited).
An adequate design would have enough phases to properly support "cross-phase" cross-validation. Deconfounding temporal noise is a basic requirement for decoding analyses of EEG and fMRI data (see e.g., leave-one-run-out CV that is effectively necessary in fMRI; in my experience, EEG is not much different, when the decoded classes are blocked in time, as here). In a journal with a typical acceptance-based review process, this would be grounds for rejection.
Please note that this issue of decoder bias would seem to weaken the rest of the downstream analyses that are based on the decoded values. For instance, if the decoders are biased, in the within-trial correlation analysis, how can we be sure that co-fluctuations along certain dimensions within their projected values are driven by signal or noise? A similar issue clouds the LMM decoding-RT correlations.
We appreciate the reviewer’s concern with the potential confound of temporally structured noise (TSN) in the EEG data. As we understand it, TSN refers to a process that the noise structure drifts over time. It follows that noise structure should be more similar for temporally closer trials and that the TSN’s bias on decoding accuracy is stronger for test trials that are closer to the training data. In the previous round of revision, we conducted a control analysis that reduced the influence of TSN by maximizing the temporal distance between training and test data (the distance between the centers of the training and test data of the same SC/SR manipulation is about 400 trials given the experimental design) and showed comparable decoding accuracy with the main results. As the reviewer finds this analysis unconvincing, we reason that the reviewer believes that the TSN has a long-term effect, such that it remains relatively stable over time and can be picked up by trials temporally distant from the training data. With this assumption and the assumption that this effect may not be linear, constructing a theoretically unbiased decoder requires perfectly counter-balanced training data (i.e., for every training trial of class A that is X trials away from the test data, there must be a training trial of all other classes that is exactly X trials away from the test data). As we were unable to achieve such a perfect design, we chose not to run an additional experiment. Instead, we focused on testing whether and how much TSN systematically biased the reported decoding accuracy.
Please note that the existence of TSN in the EEG data is not sufficient to rule that the decoding results are biased. As TSN is stronger for trials closer to each other, the idea that auto-correlation biases decoding results would predict a distance effect, such that if a test trial is closer to a training trial of the same trial type, the higher similarity in TSN between the training and test data would more strongly inflate the decoding accuracy of the test trial, resulting in a negative correlation between distance between a test trial and its closest training trial of the same type and the test trial’s decoding accuracy. To test this predicted negative correlation, in each fold and each repetition of the cross-validation reported in the SC-SC and SR-SR decoders in Fig. 4, we calculated the distance (mean=5.84 trials, SD=2.05, 5th percentile =2.87, 95th percentile=9.45, one trial = 2.4-2.6s) between each test trial and its closest training trial of the same trial type. This distance was used as the predictor to predict decoding accuracy in a linear regression. Note that even if the relation between distance and decoding accuracy is non-linear, the linear relation will be negative because the relation is monotonic (similarity in noise structure decreases monotonically with temporal distance between trials). Similarly, because the effect is monotonic, if a long-range effect exists, it should also exist in short-range and be picked up by the distance range in this analysis. The regression coefficient is averaged across cross-validation folds and repetitions for each subject to match how the decoding accuracy was reported in the main text. Finally, the averaged regression coefficient was tested against 0 using a one-sample t-test. This analysis was conducted at each time point (from -250ms to 1500ms) separately. As shown in the figure below, no time point exhibited the negative correlation as predicted by the auto-correlation account. An alternative explanation is that this result indicates that TSN remains stable over time. If this is the case, TSN will be shared by all trials and will be unable to bias decoding results. Together with the control analysis introduced previously, this new control analysis supports the notion that the decoding results are not inflated by TSN in the EEG data. We included all the control analyses in the revised manuscript (page 13-14). Please note that this analysis is specific for the present dataset and we strongly agree with the reviewer that TSN is a key confounding factor in EEG analysis in general and should be carefully addressed.
Lastly, we understand the concern with the early onset of above-chance decoding accuracy. Here, we provide an explanation: because of the blocked design (i.e., participants performed hundreds of trials with the same SC/SR associations), it is possible the participants learned the associations and used them to guide proactive cognitive control. As proactive cognitive control is anticipatory and sustained (Braver, 2012; Khan et al., 2025), it may be able to be decoded early on a trial, or even before trial onset. In the revised manuscript, we discussed this account along with the TSN issue as a limitation of the current project and directions for future research (page 24).
(2) Increase transparency in the reporting of results throughout main text.
Please do not truncate stimulus-aligned timecourses at time=0. Displaying the baseline period is very useful to identify bias, that is, to verify that stimulus-dependent conditions cannot be decoded pre-stimulus. Bias is most expected to be revealed in the baseline interval when the data are NOT baseline-corrected, which is why I previously asked to see the results omitting baseline correction. (But also note that if the decoders are biased, baseline-correcting would not remove this bias; instead, it would spread it across the rest of the epoch, while the baseline interval would, on average, be centered at zero.)
Please use a more standard p-value correction threshold, rather than Bonferroni-corrected p<0.001. This threshold is unusually conservative for this type of study. And yet, despite this conservativeness, stimulus-evoked information can be decoded from nearly every time bin, including at t=0. This does not encourage trust in the accuracy of these p-values. Instead, I suggest using permutation-based cluster correction, with corrected p<0.05. This is much more standard and would therefore allow for better comparison to many other studies.
I don't think these things should be done as control analyses, tucked away in the supplemental materials, but instead should be done as a part of the figures in the main text -- including decoding, RSA, cross-trial correlations, and RT correlations.
Thank you for your suggestions. we have added the baseline period from 200 to 0 ms prior to the stimulus onset in all the stimulus-locked analyses and tested the significance with cluster-based permutation test (cluster-forming threshold p < 0.001, cluster-level p < 0.05, (Collins & Frank, 2018)) in all the analyses including decoding, RSA, cross-trial correlations and RT correlations. The results showed similar patterns, and they are all reported in the main text (please see all the figures and page 30-32 in the main text).
Other issues:
Regarding the analysis of the within-trial correlation of RSA betas, and "Cai 2019" bias:
The correction that authors perform in the revision -- estimating the correlation within the baseline time interval and subtracting this estimate from subsequent timepoints -- assumes that the "Cai 2019" bias is stationary. This is a fairly strong assumption, however, as this bias depends not only on the design matrix, but also on the structure of the noise (see the Cai paper), which can be non-stationary. No data were provided in support of stationarity. It seems safer and potentially more realistic to assume non-stationarity.This analysis was included in the supplemental material. However, given that the correlation analysis presented in the Results is subject to the "Cai 2019" bias, it would seem to be more appropriate to replace that analysis, rather than supplement it.
Regardless, this seems to be a moot issue, given that the underlying decoders seem to be overfit to temporally structured noise (see point above regarding weakening of downstream analyses based on decoder bias).
Thank you for this important point. We now replaced the previous control analysis with a new one that does not assume stationary noise structure (page 19 in the revised manuscript). In Cai et al (2019), the source of confound is the covariance between observations. Specifically, as the observations in fMRI data are the BOLD signal at different time points, TSN can introduce covariance between nearby observations, which further biases the observed correlation between experimental conditions/trial types. In our case, the observations are decoding accuracy for different trial types. Thus, bias in the correlation may come from covariance between trial types. In this study, potential covariance between trial types includes the constrain that the decoding accuracy of all trial types adds up to 1 for a given trial (although we transformed the accuracy into logits prior to RSA, so the constrain may not hold), and the blocked design (as discussed above). Thus, to establish a baseline level of correlation between SC and SR representation strength, we took a similar shuffling approach as in Cai et al (2019) and randomly shuffled the trial types within each block. The reason to shuffle within each block is to preserve the covariance structure in the blocked design. We then repeated the same analysis using the shuffled data. The results of 10 shuffled analysis were averaged to form a baseline. Please note that (1) this control analysis was performed separately at each time point, hence removing the assumption of stationary noise structure, (2) this analysis also included as noise any covariance introduced by the proactive cognitive control guided by the learned SC and SR associations (see response to comment 1), thus it is more stringent than intended and (3) this control analysis started from decoding and was intended to provide a baseline for all downstream analysis. As shown in figures 2A, 3A, 7C and 8C, the reviewer was correct that the bias was not stationary, as the baseline of correlation coefficient varies over time. Additionally, the SC-SR representation strength correlation remained significantly above baseline between ~100 and ~ 450 ms following stimulus onset and between -180 and + 50 ms relative to response, suggesting that the noise structure (even when including potential proactive cognitive control) cannot fully explain the observed the SC-SR representation strength correlation. Considering the fact that this control analysis treated proactive control as a source of confound, this result does not necessarily contradict the absence of distance effect reported above.
Outliers and t-values:
More outliers with beta coefficients could be because the original SD estimates from the t-values are influenced more by extreme values. When you use a threshold on the median absolute deviation instead of mean +/-SD, do you still get more outliers with beta coefficients vs t-values?
Thank you for your suggestion. We calculated the proportion of outliers with a threshold of median absolute deviation (defined as values beyond median ± 5 median absolute deviation) for each subject. The outliers remained less frequent for t-values than for beta coefficients (t-values: mean = 1.08%, SD = 0.12%; beta-values: mean = 4.45%, SD = 0.28%). Based on these results and to maintain consistent with previous studies employing the methods (Cellier et al., 2022; Kikumoto & Mayr, 2020; Kikumoto et al., 2022a; Kikumoto et al., 2022b; Rangel et al., 2023), we still decided to stay with t-values.
Random slopes:
Were random slopes (by subject) for all within-subject variables included in the LMMs? If not, please include them, and report this in the Methods.
Thank you for your suggestion. The model failed to converge with random slopes of all variables. Thus, we chose not to add random slopes in the LMM. But we have added the random effects structure in the methods (see page 34).
Reviewer #2 (Public review):
Summary:
In this EEG study, Huang et al. investigated the relative contribution of two accounts to the process of conflict control, namely the stimulus-control association (SC), which refers to the phenomenon that the ratio of congruent vs. incongruent trials affects the overall control demands, and the stimulus-response association (SR), stating that the frequency of stimulus-response pairings can also impact the level of control. The authors extended the Stroop task with novel manipulation of item congruencies across blocks in order to test whether both types of information are encoded and related to behaviour. Using decoding and RSA they showed that the SC and SR representations were concurrently present in voltage signals and they also positively co-varied. In addition, the variability in both of their strengths was predictive of reaction time. In general, the experiment has a sold design and the analyses are appropriate for the research questions.
Strength:
(1) The authors used an interesting task design that extended the classic Stroop paradigm and is effective in teasing apart the relative contribution of the two different accounts regarding item-specific proportion congruency effect.
(2) Linking the strength of RSA scores with behavioural measure is critical to demonstrating the functional significance of the task representations in question.
We thank you for acknowledging our work on design and brain-behavior analysis. We have addressed all your concerns raised below point by point.
Weakness:
(1a) The distinction between Phase 2 and Phase 1&3 behavioral results, specifically the opposite effect of MC/MI in congruent trials raises some concerns with regard to the effectiveness of the ISPC manipulation. Why do RTs and error rates under MC congruent condition in Phase 2 seem to be worse than MI congruent?
Thank you for raising these issues. In Phase 1, one color set (red and blue) was assigned to the MC condition, whereas another color set (yellow and green) was assigned to the MI condition. In Phase 2, these assignments were flipped, and they were flipped back again in Phase 3. Thus, the MC condition consisted of red and blue in Phases 1 and 3 but yellow and green in Phase 2, whereas the MI condition consisted of yellow and green in Phases 1 and 3 but red and blue in Phase 2 (Fig. 1b in the manuscript). This manipulation leads to seemingly opposite patterns between Phases 1 & 3 and Phase 2.
However, when considering specific colors, the pattern is consistent across phases. In Phase 2, RTs and error rates for yellow and green (MC congruent) were worse than those for red and blue (MI congruent), which mirrors the pattern observed in Phases 1 and 3, where RTs and error rates for yellow and green (MI congruent) were worse than those for red and blue (MC congruent)
We interpreted the results in Phase 2 as reflecting a typical ISPC effect, which is defined as a smaller conflict effect in the MI condition (MI incongruent – MI congruent) compared with the MC condition (MC incongruent – MC congruent). To our knowledge, the ISPC paradigm does not impose a specific prediction regarding the relative difference between MC-congruent and MI-congruent conditions.
(1b) Could there be other factors at play here, e.g. order effect?
We agree that order effect could play a role, such that memory from Phase 1 may influence the pattern in phase 2. For example, in phase 1, yellow and green were assigned to the MI condition, and participants therefore have associated these colors with a high control state (SC) and incongruent responses (SR). These prior associations could interfere with the newly learned mappings in Phase 2, where yellow and green were reassigned to the MC congruent condition (i.e., low control state and congruent responses). As a result, memory from Phase 1 may have weakened the expected MC in phase 2. A similar effect could also apply to the MI condition. Consequently, the same condition does not show parallel performance between phase 1 and phase 2, which may lead to different patterns in the difference between MC congruent and MI congruent conditions in phase 2.
(1c) How does this potentially affect the neural analyses where trials from different phases were combined?
Thank you for the question. As we mentioned above, the order effect could slow down the newly learned associations. However, we still found the ISPC effect in each phase, suggesting that all kinds of both SC and SR associations were formed and could be applied to the decoding and the following analyses cross phases. Relatedly, there might be confounded with temporal structured noise (TSN) when the neural analyses on decoding were combined the trials from different phases. However, we have performed the control decoding analyses and distance effect tests and confirmed that our decoding results were not driven by TSN (Please see comment #1 of R1).
(1d) the manuscript does not mention whether there is counterbalancing for the color groups across participants, so far as I can tell.
Thank you for the reminder. We have balanced the color groups by randomly dividing the participants into two groups and assigning different color sets to each group. The related interpretations have been included in task overview of the revised manuscript (page 6), which reads:
“The color groups were counterbalanced across participants by red and blue as the color set of MC in one group while as the color set of MI in another group in the phase 1.”
Recommendations for the authors:
Reviewer #2 (Recommendations for the authors):
I commend the authors for addressing and clarifying my previous questions. One new comment regarding the newly added Figure 9: the response-locked behavioral correlation is much weaker compared to the stimulus-locked one, even never reaching the significance level. I think this difference should be discussed instead of simply glossing over it.
Thank you for your suggestion. We discussed the difference in the discussion of revised manuscript (page 25), which reads:
“Note that we found the negative prediction of the strength of SC and SR to RTs did not reach statistical significance with response-locked analysis as stimulus-locked analysis. It is possible that SC and SR representations have occurred before the stage of response processing, which is usually aligned with stimulus onset (Jiang et al., 2020a; Kang & Yu-Chin, 2024; Khan et al., 2025)”
References
Braver, T. S. (2012). The variable nature of cognitive control: a dual mechanisms framework. Trends Cogn Sci, 16(2), 106-113. doi:10.1016/j.tics.2011.12.010
Cellier, D., Petersen, I. T., & Hwang, K. (2022). Dynamics of Hierarchical Task Representations. J Neurosci, 42(38), 7276-7284. doi:10.1523/JNEUROSCI.0233-22.2022
Collins, A. G., & Frank, M. J. (2018). Within- and across-trial dynamics of human EEG reveal cooperative interplay between reinforcement learning and working memory. Proceedings of the National Academy of Sciences, 115(10), 2502-2507. doi:10.1073/pnas.1720963115
Khan, A. U., Hoy, C. W., Anderson, K. L., Piai, V., King-Stephens, D., Laxer, K. D., . . . Bentley, J. N. (2025). Neural dynamics of proactive and reactive cognitive control in medial and lateral prefrontal cortex. iScience, 28(9), 113375. doi:10.1016/j.isci.2025.113375
Kikumoto, A., & Mayr, U. (2020). Conjunctive representations that integrate stimuli, responses, and rules are critical for action selection. Proc Natl Acad Sci 117(19), 10603-10608. doi:10.1073/pnas.1922166117
Kikumoto, A., Mayr, U., & Badre, D. (2022a). The role of conjunctive representations in prioritizing and selecting planned actions. Elife, 11. doi:10.7554/eLife.80153
Kikumoto, A., Sameshima, T., & Mayr, U. (2022b). The Role of Conjunctive Representations in Stopping Actions. Psychol Sci, 33(2), 325-338. doi:10.1177/09567976211034505
Rangel, B. O., Hazeltine, E., & Wessel, J. R. (2023). Lingering Neural Representations of Past Task Features Adversely Affect Future Behavior. J Neurosci, 43(2), 282-292. doi:10.1523/JNEUROSCI.0464-22.2022
-
eLife Assessment
This useful study uses creative scalp EEG decoding methods to demonstrate that two forms of learned associations in a Stroop task are dissociable, despite sharing similar temporal dynamics. The evidence supporting the conclusions is solid, although it could be further strengthened with a modified experimental design. This paper would be of interest to researchers studying cognitive control and adaptive behavior.
-
Reviewer #2 (Public review):
Summary:
In this EEG study, Huang et al. investigated the relative contribution of two accounts to the process of conflict control, namely the stimulus-control association (SC), which refers to the phenomenon that the ratio of congruent vs. incongruent trials affects the overall control demands, and the stimulus-response association (SR), stating that the frequency of stimulus-response pairings can also impact the level of control. The authors extended the Stroop task with novel manipulation of item congruencies across blocks in order to test whether both types of information are encoded and related to behaviour. Using decoding and RSA they showed that the SC and SR representations were concurrently present in voltage signals and they also positively co-varied. In addition, the variability in both of their …
Reviewer #2 (Public review):
Summary:
In this EEG study, Huang et al. investigated the relative contribution of two accounts to the process of conflict control, namely the stimulus-control association (SC), which refers to the phenomenon that the ratio of congruent vs. incongruent trials affects the overall control demands, and the stimulus-response association (SR), stating that the frequency of stimulus-response pairings can also impact the level of control. The authors extended the Stroop task with novel manipulation of item congruencies across blocks in order to test whether both types of information are encoded and related to behaviour. Using decoding and RSA they showed that the SC and SR representations were concurrently present in voltage signals and they also positively co-varied. In addition, the variability in both of their strengths was predictive of reaction time. In general, the experiment has an innovative design and the analytical choices are appropriate and the evidence supporting the conclusions are overall solid after taking consideration the control analyses the authors have provided, although within limits of their study design.
Strength:
(1) The authors used an interesting task design that extended the classic Stroop paradigm and is effective in teasing apart the relative contribution of the two different accounts regarding item-specific proportion congruency effect.
(2) Linking strength of RSA scores with behavioural measure is critical to demonstrating the functional significance of the task representations in question.
Comments on revised version.
I appreciate the tireless effort the authors have presented to provide extra control analyses, however, on the other hand I do wish to remind them that sometimes limitations of one study is better addressed by a new study with improved design. There is very good reason why orthogonalization is critical to separating confounding influencing factors which the current study did not completely achieve. Reviewer 1's suggestion on alternative designs is certainly worth considering, and I encourage the authors to continue working on perfecting the experimental design in future work.
-
Author response:
The following is the authors’ response to the previous reviews
eLife Assessment
This useful study uses creative scalp EEG decoding methods to attempt to demonstrate that two forms of learned associations in a Stroop task are dissociable, despite sharing similar temporal dynamics. However, the evidence supporting the conclusions is incomplete due to concerns with the experimental design and methodology. This paper would be of interest to researchers studying cognitive control and adaptive behavior, if the concerns raised in the reviews can be addressed satisfactorily.
We thank the editors and the reviewers for their positive assessment and constructive feedback on our work. We also thank the editor for communicating with reviewer #1 regarding our thoughts on their comments. We hence revised the manuscript based the new …
Author response:
The following is the authors’ response to the previous reviews
eLife Assessment
This useful study uses creative scalp EEG decoding methods to attempt to demonstrate that two forms of learned associations in a Stroop task are dissociable, despite sharing similar temporal dynamics. However, the evidence supporting the conclusions is incomplete due to concerns with the experimental design and methodology. This paper would be of interest to researchers studying cognitive control and adaptive behavior, if the concerns raised in the reviews can be addressed satisfactorily.
We thank the editors and the reviewers for their positive assessment and constructive feedback on our work. We also thank the editor for communicating with reviewer #1 regarding our thoughts on their comments. We hence revised the manuscript based the new feedback from reviewer #1. Please see below our responses to each comment raised in the reviews.
Public Reviews:
Reviewer #1 (Public review):
Summary:
This study focuses on characterizing the EEG correlates of item-specific proportion congruency effects. In particular, two types of learned associations are studied. One association involves associations between stimulus features and control states (SC), and the other involves stimulus features and responses (SR). Decoding methods are used to identify time-resolved SC and SR correlates.
The authors conclude that SC and SR associations can independently and simultaneously guide behavior. This conclusion is based on results showing that SC and SR correlates are (1) not entirely overlapping in cross-decoding, (2) simultaneously observed on average over trials, (3) independently correlate with RT, and (4) have a positive within-trial correlation.
Strengths:
Fearless, creative use of EEG decoding to test tricky hypotheses regarding latent associations.
Nice idea to orthogonalize ISPC condition (MC/MI) from stimulus features.
Thank you for acknowledging the strength in EEG decoding and design. We have addressed all your concerns raised below point by point.
In my view, the ability to address this issue with additional analyses is relatively limited. I cannot think of a solid way to escape this issue in the present design. Adding a nuisance regressor to their RSA regression, which I suggested in my previous response, may reduce the bias, but the efficacy of this would be limited to controlling only a certain kind of phase-dependent confound (a 'main effect' component of study phase, i.e., one that is constant across other conditions; see next message for discussion).
Rather than new analyses, I think a more straightforward revision might be to modify the conclusions advanced in the paper, so that they are more solidly supported by the design and evidence. In my opinion, this design is ill-posed to solidly identify SC and SR representations. As a result, I think that any framing that alleviates pressure on this design to yield 'solid' evidence for identification of SC and SR representations, and instead emphasizes stronger areas of this work, would be constructive.
For example, one potential framing is to advance the idea of SC and SR representations, and discuss an idealized design that could identify them by orthogonalizing stimulus features from ISPC, which are genuinely novel and useful ideas. The current design could then be presented as an opportunistic or initial case study of testing this question, while acknowledging its limitation upfront. The goal here would be to frame the study in a way that allows for the results to be presented with an appropriate grain of salt, while also illustrating the authors thoughtfulness and creativity in devising analyses to test for latent associative representations. In this case the 'solid' label would reference the authors' reasoning and analyses rather than design and conclusions.
I only intend this example as an illustration; there may be several ways of framing this paper so that it is on more 'solid' ground, and I don't want to dictate how exactly authors should write their paper.
Nonetheless I think this issue is important, not only to avoid faulty inference, but also to avoid establishing counterproductive precedents in this field. For example, if students read a paper whose conclusions are labeled "solid" but that nevertheless has critical flaws in its design, then those students may be misled in their own work. But if the flaws were discussed transparently and critically, and the strength of the conclusions were de-emphasized relative to other aspects of the paper, students may not only be inspired by the ideas developed in the paper, but also come away with knowledge about the issues of experimental design.
Discussion of the weaknesses in the conclusions and an additional potential analysis:
The key goal of this study is to identify SC/SR representations, which requires decoupling stimulus features from item-specific proportion congruency (ISPC), but the study-phase confound contaminates this decoupling. I think this impacts both their cross-phase decoding and RSA analyses.
In their results (lines 139-144):
"This standard ISPC manipulation can test whether neural representations of controlled and non-controlled information are wrapped on the same trial by combing with the following EEG analysis (See Methods). However, it potentially mixes color identity with SC, word identity with SR, and the ISPC between SC and SR. To deconfound these factors when estimating SC and SR association representations on each trial, we modified this paradigm by flipping the ISPC contingencies across different phases of the task."
SC/SR representations are higher-order conjunctive classes, formed by the interaction of lower order variables (Color, Word, and ISPC). This means that successfully identifying these representations relies on demonstrating that each class can be reliably individuated from every other class in a manner that cannot be explained by (1) representation of shared lower-order features, such as stimulus color or response, and (2) trivial nuisance factors such as study phase. However, in this design, the trivial factor of study phase is strongly confounded with the ISPC contingency flip.
Regarding RSA: If study phase indeed leads to trivial separability, it seems that similarity among conditions within the same phase would be inflated because the study phase does not appear in the RSA model (Figure 12). In which case, the SC/SR coefficients would be inflated, as the SC and SR models are entirely within-phase.
Nevertheless, an additional control analysis may be possible here. Looking at this regressor set, it seems possible to me to fit a model where the predominant phase is entered as an additional covariate. (If I am reading this correctly, phase would appear as a 2x2 block-diagonal matrix). I suggested this in my last review, but in their recent letter, authors refused. I do not understand why, as I think this regressor set should be identifiable, but perhaps I am wrong here.
That being said, I do not think adding this nuisance covariate would fully solve the issue. The lower-order regressors (Color, Word, ISPC) are defined as the EEG responses shared across phases of the study. To interpret the higher-order SR/SC coefficients, the lower-order components must be fully partialled out. But the putative impact of study phase contaminates this interpretation, as study phase could trivially decrease the similarity of lower-order terms (e.g., decreasing Color similarity between phase 2 vs 3). In which case, the partialling would be expected to be incomplete.
This incomplete partialling is the RSA analogue of the issue in interpreting cross-phase decoding discussed above. As there, so too here I do not see a solid way around it in the present design. This is why in my previous review I referred to the addition of a phase covariate in the RSA regression as a "band-aid": it controls for some problems (main effect of phase), but not all (interactions of phase and lower-order terms).
To summarize, I think that RSA would offer an additional opportunity to control for this potential confound, albeit in a limited sense (study phase effects that are consistent across conditions). But in a more general and rigorous sense, to me, the SC and SR terms in the RSA regression also seem susceptible to the same weakness as the cross-phase decoding analysis.
We thank the reviewer for taking the additional time and effort to provide the new comments. Following the reviewer’s suggestion, we revised the language regarding the conclusions of this project (page 2,5,27-28) and explicitly discussed the weaknesses of the design on decoding and outline a possible solution for future studies in the Discussion section:
“A limitation of the current design is that in theory temporally structured noise (e.g., autocorrelation in EEG data) may bias the decoding accuracy due to the blocked design. Although the present data provided no evidence that the decoding results in this study were biased by temporally structured noise, future studies should aim to develop experimental designs that eliminate this potential confound at the source. One potential solution would be to introduce additional phases flipping ISPC manipulations. At the same time, enough trials must be included in each phase to ensure the strength of the ISPC effect within each phase. A careful balance between session number and length will be helpful to optimize the duration of such a design.”
As eLife also publishes review report, below we also summarize the three control analyses we ran and our reasoning of how they (would) address the issue of temporally structured noise for interested readers to assess:
We acknowledge the theoretical issue of temporally structured noise (TSN) in our design when classes were decoded across different phases. However, the key question for the current data is whether there is empirical evidence that the decoding results were actually driven by TSN. To clarify this issue, we summarize several lines of evidence suggesting that the decoding results were not attributable to TSN:
(1) Split-half cross-validation. We split the EEG data from Phase 2 and the combined Phases 1 and 3 into chronological first and second halves. Phases 1 and 3 were combined because they shared the same MC and MI assignments. This resulted in four possible combinations, each consisting of eight classes drawn from different phases: combination 1 included the first half of Phase 2 and the first half of Phase 3; combination 2 included the first half of Phase 2 and the second half of Phase 3; combination 3 included the second half of Phase 2 and the first half of Phase 3; and combination 4 included the second half of Phase 2 and the second half of Phase 3. We trained the decoders on one combination and tested them on another and then averaged the decoding results across all possible training-test assignments. The similar decoding patterns observed across these analyses (Fig. 6a,b) further confirmed that the decoding results were not driven by TSN.
This analysis is conceptually similar to the “cross-phase” decoding analysis suggested by the reviewer in the first round of review. We also performed an additional distance-based control analysis (see below) to further test whether the decoding results could be explained by TSN, without imposing the constraint used in the split-half cross-validation that trials from the two phases had to fall within a 400-trial window.
(2) Distance analysis. We predicted that if a test trial is closer to a training trial of the same trial type, the higher similarity in TSN between the training and test data would more strongly inflate the decoding accuracy of the test trial, resulting in a negative correlation between distance between a test trial and its closest training trial of the same type and the test trial’s decoding accuracy. However, we did not observe such a negative pattern (Fig. 6c). Note that this distance was defined with respect to trials of the same type, rather than absolute chronological time.
(3) Shuffled analysis. If the decoding results were primarily driven by TSN, either at a short-term or long-term timescale, then shuffling the condition labels within each mini block should preserve the TSN structure present in the real data. In that case, the decoding results from shuffled data should not differ from those observed from real data. However, we found the significant difference between real data and shuffled data as shown in Author response images.
Author response image 1.
Shuffling analyses with stimulus-locked data support separable SC and SR subspace. (a) Group average decoding accuracy of all 16 experimental conditions as a function of time after stimulus onset. Squares below the lines indicate the significant time points between real data and shuffled data (cluster-based permutation test, cluster-forming threshold p < 0.001, cluster-level p < 0.05). (b) Group average t values of representational strength for each factor over time. Squares below the lines indicate the significant time points between real data and shuffled data (cluster-based permutation test, cluster-forming threshold p < 0.001, cluster-level p < 0.05). (c) SC and SR association results from Fig. 1b.

Author response image 2.
Shuffling analyses with response-locked data support separable SC and SR subspace. (a) Group average decoding accuracy of all 16 experimental conditions as a function of time after stimulus onset. Squares below the lines indicate the significant time points between real data and shuffled data (cluster-based permutation test, cluster-forming threshold p < 0.001, cluster-level p < 0.05). (b) Group average t values of representational strength for each factor over time. Squares below the lines indicate the significant time points between real data and shuffled data (cluster-based permutation test, cluster-forming threshold p < 0.001, cluster-level p < 0.05). (c) SC and SR association results from Fig. 2b.

We thank the reviewer for the suggestion on RSA with phase. There are some concerns for this analysis:
First, we think that the suggested analysis may be difficult to interpret. Because the SC and SR conditions differ across phases. Regressing out phase in RSA could also remove SC and SR information.
Second, based on the reviewer’s comment, we understand that the suggested analysis may still not provide a clear falsifiable criterion for determining whether the results could be driven by the theoretical TSN issue inherent in the design.
Third, the three control analyses we have performed examine this issue from different perspectives and collectively provide no evidence that the results were driven by TSN.
Other readers may, like me, be puzzled by the selection of this particular experimental design to test this question of SC and SR coding, given the temporal confound among SC/SR classes, and given that there would seem to be many possible designs that are less confounded. For example, why not use a design where ISPC was swapped/shuffled several more times within each subject, so that PHASE is more orthogonal to long-timescale noise? Isn't ISPC learning fast enough to support learning phases shorter than 700 trials? Such readers would likely appreciate a frank discussion of this dilemma, and a motivation for the choice of the present design, within the manuscript.
Thank you for your suggestion regarding the design. It is possible that the (re-)learning of ISPC can be fast. That said, enough trials are required to obtain a robust ISPC effect for each phase after the ISPC flips. Given that the EEG scanning (not including capping) in current design was about 1.5 hours, it is impractical to have both more sessions for a more orthogonal design and long sessions for robust within-session ISPC effects. We chose to maximize the latter because flipped behavioral ISPC effect in each session is the basis for the following EEG analysis. We have included the reviewer’s suggestion as a potential design solution for future studies in the Discussion section mentioned above on page 27.
Pre-stimulus coding:
To explain the apparent pre-stimulus coding of several task variables, the newest version of the manuscript proposes that subjects were proactively coding these variables via predictive mechanisms. This is an interesting account of item-specific control. It is also surprising, given that item-specific control mechanisms are typically conceptualized as reactive or stimulus-driven phenomena. But I think support for a proactive control account was incomplete. The mechanistic logic was not presented, and no hypotheses under this account were developed or tested. So I would suggest pinning down some hypotheses here and actually putting this account to the test.
Thank you for raising this important point. Although ISPC effects are considered reactive, in our design the long sessions may create a temporal context for the participants to differentiate the current control demand linked to each color. The maintenance of such contextual information needs to span across trials, leading to pre-stimulus coding that proactively guides the control demand for each color. This claim is not central to this manuscript, which investigates whether SC and SR representations simultaneously guide behavior. Additionally, we do not think the current design is well-equipped to test this hypothesis because the pre-stimulus onset is the only supporting evidence. In the revised manuscript, we discussed this as a future research direction and proposed a design that aims at better isolating proactive control signal on page 25.
Random slopes were omitted due to convergence failure, but this can inflate false positive inferences (e.g., Barr et al. 2013), and doesn't really motivate a minimal model. I'd suggest trying a slightly reduced model (e.g., drop correlations via `slope || subject`) using buildMer automated selection, or switching to brms.
We indeed tried both the full model of random effects (i.e., considering covariance between all slopes and intercept) and a reduced model without any covariance (i.e., listing each random slope separately without intercept in lme4). However, neither model converged at all time points.
Reviewer #2 (Public review):
Summary:
In this EEG study, Huang et al. investigated the relative contribution of two accounts to the process of conflict control, namely the stimulus-control association (SC), which refers to the phenomenon that the ratio of congruent vs. incongruent trials affects the overall control demands, and the stimulus-response association (SR), stating that the frequency of stimulus-response pairings can also impact the level of control. The authors extended the Stroop task with novel manipulation of item congruencies across blocks in order to test whether both types of information are encoded and related to behaviour. Using decoding and RSA they showed that the SC and SR representations were concurrently present in voltage signals and they also positively co-varied. In addition, the variability in both of their strengths was predictive of reaction time. In general, the experiment has a solid design and the analyses are appropriate for the research questions.
Strengths:
(1) The authors used an interesting task design that extended the classic Stroop paradigm and is effective in teasing apart the relative contribution of the two different accounts regarding item-specific proportion congruency effect.
(2) Linking the strength of RSA scores with behavioural measure is critical to demonstrating the functional significance of the task representations in question.
We thank you for acknowledging our work on design and brain-behavior analysis. We have addressed your concerns raised below.
Weaknesses:
I still have some doubts on the effectiveness of the experimental manipulation on Phase 2: although the ISPC effect is still present, it is much weaker in comparison, suggesting the participants did not learn the contingency statistics in Phase 2 as well as they did in the other phases, due to either the lingering effect of the previous phase or an inherent bias towards one color pairs. Perhaps by separately plotting the earlier and later blocks of Phase 2 any difference can be revealed if it exists. This behavioral difference could result in unequal levels of SC/SR representation across phases, which may raise problems when data were combined for analyses that assume the neural effects are equivalent.
Thank you for your concern about this important issue. We agree with the reviewer that the true SR/SC levels may not be equivalent between Phase 2 and Phase 1/3. Nevertheless, because the manipulation of ISPC is binary, the decoders were trained to test whether the neural signals represent the two levels of ISPC (i.e., a higher vs. a lower level) differ systematically. The decoding analysis does not require that the neural effects of SC and SR must be numerically equivalent between phases (i.e., it is not necessary that the two levels are equidistant from the center point of SC/SR. Indeed, the decoding analysis only requires that the two levels are different). For example, if the ISPC level ranges from -1 to 1 and the EEG signals can reliably decode ISPC levels of -0.5 and 0.7 (i.e., two unequal levels), it can still be treated as supporting evidence that ISPC levels are encoded in the EEG signals. The same logic applies to the representational subspace analysis. As to the RSA, as can be seen in Fig. 12, the regressors are also binary, encoding whether two experimental conditions share the same SC/SR level without assuming equivalent neural effects. Thus, we argue that the reported decoding and RSA can still test the encoding of SR and SC. We discussed this issue on page 24.
Following the reviewer’s comment, we plotted the ISPC effects in first and second half of Phase 2 separately (the figure below). We also tested whether the ISPC effects differ qualitatively between the two halves using a 3-way ANOVAs separately on RT and Error rate. The results showed that the time (the first half vs. the second half) × Congruency × ISPC interaction was not significant for either RT data (F(1,39) = 3.40, p > 0.05) or error rate (F(1,39) = 2.49, p > 0.05), suggesting that ISPC effect did not systematically change over time in Phase 2 See Supplementary Figure 9.
-
Authors published a paper in Biorxiv, they used PsychoPy in the study. Including #RRIDs will make this less ambiguous. SciScore made a table with this resource, see “Automated Services” module (download as csv, xml or #jats) #RRID #methodsmatter
-

-
-
eLife Assessment
This useful study uses creative scalp EEG decoding methods to attempt to demonstrate that two forms of learned associations in a Stroop task are dissociable, despite sharing similar temporal dynamics. However, the evidence supporting the conclusions is incomplete due to concerns with the experimental design and methodology. This paper would be of interest to researchers studying cognitive control and adaptive behavior, if the concerns raised in the reviews can be addressed satisfactorily.
-
Reviewer #1 (Public review):
Summary:
This study focuses on characterizing the EEG correlates of item-specific proportion congruency effects. Two types of learned associations are characterized, one being associations between stimulus features and control states (SC), and the other being stimulus features and responses (SR). Decoding methods are used to identify time-resolved SC and SR correlates, which are used to test properties of their dynamics.
The conclusion is reached that SC and SR associations can independently and simultaneously guide behavior. This conclusion is based on results showing SC and SR correlates are: (1) not entirely overlapping in cross-decoding; (2) simultaneously observed on average over trials in overlapping time bins; (3) independently correlate with RT; and (4) have a positive within-trial correlation.
Streng…
Reviewer #1 (Public review):
Summary:
This study focuses on characterizing the EEG correlates of item-specific proportion congruency effects. Two types of learned associations are characterized, one being associations between stimulus features and control states (SC), and the other being stimulus features and responses (SR). Decoding methods are used to identify time-resolved SC and SR correlates, which are used to test properties of their dynamics.
The conclusion is reached that SC and SR associations can independently and simultaneously guide behavior. This conclusion is based on results showing SC and SR correlates are: (1) not entirely overlapping in cross-decoding; (2) simultaneously observed on average over trials in overlapping time bins; (3) independently correlate with RT; and (4) have a positive within-trial correlation.
Strengths:
Fearless, creative use of EEG decoding to test tricky hypotheses regarding latent associations.
Nice idea to orthogonalize ISPC condition (MC/MI) from stimulus features.
Weaknesses:
I still have my concern from the first round that the decoders are overfit to temporally structured noise. As I wrote before, the SC and SR classes are highly confounded with phase (chunk of session). I do not see how the control analyses conducted in the revision adequately deal with this issue.
In the figures, there are several hints that these decoders are biased. Unfortunately, the figures are also constructed in such a way that hides or diminishes the salience of the clues of bias. This bias and lack of transparency discourage trust in the methods and results.
I have two main suggestions:
(1) Run a new experiment with a design that properly supports this question.
I don't make this suggestion lightly, and I understand that it may not be feasible to implement given constraints; but I feel that this suggestion is warranted. The desired inferences rely on successful identification of SC and SR representations. Solidly identifying SC and SR representations necessitates an experimental design wherein these variables are sufficiently orthogonalized, within-subject, from temporally structured noise. The experimental design reported in this paper unfortunately does not meet this bar, in my opinion (and the opinion of a colleague I solicited).
An adequate design would have enough phases to properly support "cross-phase" cross-validation. Deconfounding temporal noise is a basic requirement for decoding analyses of EEG and fMRI data (see e.g., leave-one-run-out CV that is effectively necessary in fMRI; in my experience, EEG is not much different, when the decoded classes are blocked in time, as here). In a journal with a typical acceptance-based review process, this would be grounds for rejection.
Please note that this issue of decoder bias would seem to weaken the rest of the downstream analyses that are based on the decoded values. For instance, if the decoders are biased, in the within-trial correlation analysis, how can we be sure that co-fluctuations along certain dimensions within their projected values are driven by signal or noise? A similar issue clouds the LMM decoding-RT correlations.
(2) Increase transparency in the reporting of results throughout main text.
Please do not truncate stimulus-aligned timecourses at time=0. Displaying the baseline period is very useful to identify bias, that is, to verify that stimulus-dependent conditions cannot be decoded pre-stimulus. Bias is most expected to be revealed in the baseline interval when the data are NOT baseline-corrected, which is why I previously asked to see the results omitting baseline correction. (But also note that if the decoders are biased, baseline-correcting would not remove this bias; instead, it would spread it across the rest of the epoch, while the baseline interval would, on average, be centered at zero.)
Please use a more standard p-value correction threshold, rather than Bonferroni-corrected p<0.001. This threshold is unusually conservative for this type of study. And yet, despite this conservativeness, stimulus-evoked information can be decoded from nearly every time bin, including at t=0. This does not encourage trust in the accuracy of these p-values. Instead, I suggest using permutation-based cluster correction, with corrected p<0.05. This is much more standard and would therefore allow for better comparison to many other studies.
I don't think these things should be done as control analyses, tucked away in the supplemental materials, but instead should be done as a part of the figures in the main text -- including decoding, RSA, cross-trial correlations, and RT correlations.
Other issues:
Regarding the analysis of the within-trial correlation of RSA betas, and "Cai 2019" bias:
The correction that authors perform in the revision -- estimating the correlation within the baseline time interval and subtracting this estimate from subsequent timepoints -- assumes that the "Cai 2019" bias is stationary. This is a fairly strong assumption, however, as this bias depends not only on the design matrix, but also on the structure of the noise (see the Cai paper), which can be non-stationary. No data were provided in support of stationarity. It seems safer and potentially more realistic to assume non-stationarity.
This analysis was included in the supplemental material. However, given that the correlation analysis presented in the Results is subject to the "Cai 2019" bias, it would seem to be more appropriate to replace that analysis, rather than supplement it.
Regardless, this seems to be a moot issue, given that the underlying decoders seem to be overfit to temporally structured noise (see point above regarding weakening of downstream analyses based on decoder bias).
Outliers and t-values:
More outliers with beta coefficients could be because the original SD estimates from the t-values are influenced more by extreme values. When you use a threshold on the median absolute deviation instead of mean +/-SD, do you still get more outliers with beta coefficients vs t-values?
Random slopes:
Were random slopes (by subject) for all within-subject variables included in the LMMs? If not, please include them, and report this in the Methods.
-
Reviewer #2 (Public review):
Summary:
In this EEG study, Huang et al. investigated the relative contribution of two accounts to the process of conflict control, namely the stimulus-control association (SC), which refers to the phenomenon that the ratio of congruent vs. incongruent trials affects the overall control demands, and the stimulus-response association (SR), stating that the frequency of stimulus-response pairings can also impact the level of control. The authors extended the Stroop task with novel manipulation of item congruencies across blocks in order to test whether both types of information are encoded and related to behaviour. Using decoding and RSA they showed that the SC and SR representations were concurrently present in voltage signals and they also positively co-varied. In addition, the variability in both of their …
Reviewer #2 (Public review):
Summary:
In this EEG study, Huang et al. investigated the relative contribution of two accounts to the process of conflict control, namely the stimulus-control association (SC), which refers to the phenomenon that the ratio of congruent vs. incongruent trials affects the overall control demands, and the stimulus-response association (SR), stating that the frequency of stimulus-response pairings can also impact the level of control. The authors extended the Stroop task with novel manipulation of item congruencies across blocks in order to test whether both types of information are encoded and related to behaviour. Using decoding and RSA they showed that the SC and SR representations were concurrently present in voltage signals and they also positively co-varied. In addition, the variability in both of their strengths was predictive of reaction time. In general, the experiment has a sold design and the analyses are appropriate for the research questions.
Strength:
(1) The authors used an interesting task design that extended the classic Stroop paradigm and is effective in teasing apart the relative contribution of the two different accounts regarding item-specific proportion congruency effect.
(2) Linking the strength of RSA scores with behavioural measure is critical to demonstrating the functional significance of the task representations in question.
Weakness:
(1) The distinction between Phase 2 and Phase 1&3 behavioral results, specifically the opposite effect of MC/MI in congruent trials raises some concerns with regard to the effectiveness of the ISPC manipulation. Why do RTs and error rates under MC congruent condition in Phase 2 seem to be worse than MI congruent? Could there be other factors at play here, e.g. order effect? How does this potentially affect the neural analyses where trials from different phases were combined? Also, the manuscript does not mention whether there is counterbalancing for the color groups across participants, so far as I can tell.
-
Author response:
The following is the authors’ response to the original reviews.
eLife Assessment
This useful study uses creative scalp EEG decoding methods to attempt to demonstrate that two forms of learned associations in a Stroop task are dissociable, despite sharing similar temporal dynamics. However, the evidence supporting the conclusions is incomplete due to concerns with the experimental design and methodology. This paper would be of interest to researchers studying cognitive control and adaptive behavior, if the concerns raised in the reviews can be addressed satisfactorily.
We thank the editors and the reviewers for their positive assessment of our work and for providing us with an opportunity to strengthen this manuscript. Please see below our responses to each comment raised in the reviews.
Public Reviews:
Reviewer #1 …
Author response:
The following is the authors’ response to the original reviews.
eLife Assessment
This useful study uses creative scalp EEG decoding methods to attempt to demonstrate that two forms of learned associations in a Stroop task are dissociable, despite sharing similar temporal dynamics. However, the evidence supporting the conclusions is incomplete due to concerns with the experimental design and methodology. This paper would be of interest to researchers studying cognitive control and adaptive behavior, if the concerns raised in the reviews can be addressed satisfactorily.
We thank the editors and the reviewers for their positive assessment of our work and for providing us with an opportunity to strengthen this manuscript. Please see below our responses to each comment raised in the reviews.
Public Reviews:
Reviewer #1 (Public review):
Summary:
This study focuses on characterizing the EEG correlates of item-specific proportion congruency effects. In particular, two types of learned associations are characterized. One being associations between stimulus features and control states (SC), and the other being stimulus features and responses (SR). Decoding methods are used to identify SC and SR correlates and to determine whether they have similar topographies and dynamics.
The results suggest SC and SR associations are simultaneously coactivated and have shared topographies, with the inference being that these associations may share a common generator.
Strengths:
Fearless, creative use of EEG decoding to test tricky hypotheses regarding latent associations. Nice idea to orthogonalize the ISPC condition (MC/MI) from stimulus features.
Thank you for acknowledging the strength in EEG decoding and design. We have addressed all your concerns raised below point by point.
Weaknesses:
(1a) I'm relatively concerned that these results may be spurious. I hope to be proven wrong, but I would suggest taking another look at a few things.
While a nice idea in principle, the ISPC manipulation seems to be quite confounded with the trial number. E.g., color-red is MI only during phase 2, and is MC primarily only during Phase 3 (since phase 1 is so sparsely represented). In my experience, EEG noise is highly structured across a session and easily exploited by decoders. Plus, behavior seems quite different between Phase 2 and Phase 3. So, it seems likely that the classes you are asking the decoder to separate are highly confounded with temporally structured noise.
I suggest thinking of how to handle this concern in a rigorous way. A compelling way to address this would be to perform "cross-phase" decoding, however I am not sure if that is possible given the design.
Thank you for raising this important issue. To test whether decoding might be confounded by temporally structured noise, we performed a control decoding analysis. As the reviewer correctly pointed out, cross-phase decoding is not possible due to the experimental design. Alternatively, to maximize temporal separation between the training and test data, we divided the EEG data in phase 2 and phase 1&3 into the first and second half chronologically. Phase 1 and 3 were combined because they share the same MC and MI assignments. We then trained the decoders on one half and tested them on the other half. Finally, we averaged the decoding results across all possible assignments of training and test data. The similar patterns (Supplementary Fig.1) observed confirmed that the decoding results are unlikely to be driven by temporally structured noise in the EEG data. The clarification has been added to page 13 of the revised manuscript.
(1b) The time courses also seem concerning. What are we to make of the SR and SC timecourses, which have aggregate decoding dynamics that look to be <1Hz?
As detailed in the response to your next comment, some new results using data without baseline correction show a narrower time window of above-chance decoding. We speculate that the remaining results of long-lasting above-chance decoding could be attributed to trials with slow responses (some responses were made near the response deadline of 1500 ms). Additionally, as shown in Figure 6a, the long-lasting above-chance decoding seems to be driven by color and congruency representations. Thus, it is also possible that the binding of color and congruency contributes to decoding. This interpretation has been added to page 17 of the revised manuscript.
(1c) Some sanity checks would be one place to start. Time courses were baselined, but this is often not necessary with decoding; it can cause bias (10.1016/j.jneumeth.2021.109080), and can mask deeper issues. What do things look like when not baselined? Can variables be decoded when they should not be decoded? What does cross-temporal decoding look like - everything stable across all times, etc.?
As the reviewer mentioned, baseline-corrected data may introduce bias to the decoding results. Thus, we cited the van Driel et al (2021) paper in the revised manuscript to justify the use of EEG data without baseline-correction in decoding analysis (Page 27 of the revised manuscript), and re-ran all decoding analysis accordingly. The new results revealed largely similar results (Fig. 2, 4, 6 and 8 in the revised manuscript) with the following exceptions: narrower time window for separatable SC subspace and SR subspace (Fig. 4b), narrower time window for concurrent representations of SC and SR (Fig. 6a-b), and wider time window for the correlations of SC/SR representations with RTs (Fig. 8).
(2) The nature of the shared features between SR and SC subspaces is unclear.
The simulation is framed in terms of the amount of overlap, revealing the number of shared dimensions between subspaces. In reality, it seems like it's closer to 'proportion of volume shared', i.e., a small number of dominant dimensions could drive a large degree of alignment between subspaces.
What features drive the similarity? What features drive the distinctions between SR and SC? Aside from the temporal confounds I mentioned above, is it possible that some low-dimensional feature, like EEG congruency effect (e.g., low-D ERPs associated with conflict), or RT dynamics, drives discriminability among these classes? It seems plausible to me - all one would need is non-homogeneity in the size of the congruency effect across different items (subject-level idiosyncracies could contribute: 10.1016/j.neuroimage.2013.03.039).
Thank you for this question. To test what dimensions are shared between SC and SR subspaces, we first identify which factors can be shared across SC and SR subspaces. For SC, the eight conditions are the four colors × ISPC. Thus, the possible shared dimensions are color and ISPC. Additionally, because the four colors and words are divided into two groups (e.g., red-blue and green-yellow, counterbalanced across subjects, see Methods), the group is a third potential shared dimension. Similarly, for SR decoders, potential shared dimensions are word, ISPC and group. Note that each class in SC and SR decoders has both congruent and incongruent trials. Thus, congruency is not decodable from SC/SR decoders and hence unlikely to be a shared dimension in our analysis. To test the effect of sharing for each of the potential dimensions, we performed RSA on decoding results of the SC decoder trained on SR subspace (SR | SC) (Supplementary Fig. 4a) and the SR decoder trained on SC subspace (SC | SR) (Supplementary Fig. 4b), where the decoders indicated the decoding accuracy of shared SC and SR representations. In the SC classes of SR | SC, word red and blue were mixed within the same class, same were word yellow and green. The similarity matrix for “Group” of SR | SC (Supplementary Fig. 4a) shows the comparison between two word groups (red & blue vs. yellow & green). The similarity matrix for “Group” of SC | SR (Supplementary Fig. 4b) shows the comparison between two color groups (red & blue vs. yellow & green).
The RSA results revealed that the contributions of group to the SC decoder (Supplementary Fig. 5a) and the SR decoder (Supplementary Fig. 5b) were significant. Meanwhile, a wider time window showed significant effect of color on the SC decoder (approximately 100 - 1100 ms post-stimulus onset, Supplementary Fig. 5a) and a narrower time window showed significant effect of word on SR decoder (approximately 100 - 500 ms post-stimulus onset, Supplementary Fig. 5b). However, we found no significant effect of ISPC on either SC or SR decoders. We also performed the same analyses on response-locked data from the time window -800 to 200 ms. The results showed shared representation of color in the SC decoder (Supplementary Fig. 5c) and group in both decoders (Supplementary Fig. 5c-d). Overall, the above results demonstrated that color, word and group information are shared between SC and SR subspaces.
Lastly, we would like to stress that our main hypothesis for the cross-subspace decoding analysis is that SR and SC subspaces are not identical. This hypothesis was supported by lower decoding accuracy for cross-subspace than within-subspace decoders and enables following analyses that treated SC and SR as separate representations.
We have added the interpretation to page 13-14 of the revised manuscript.
(3) The time-resolved within-trial correlation of RSA betas is a cool idea, but I am concerned it is biased. Estimating correlations among different coefficients from the same GLM design matrix is, in general, biased, i.e., when the regressors are non-orthogonal. This bias comes from the expected covariance of the betas and is discussed in detail here (10.1371/journal.pcbi.1006299). In short, correlations could be inflated due to a combination of the design matrix and the structure of the noise. The most established solution, to cross-validate across different GLM estimations, is unfortunately not available here. I would suggest that the authors think of ways to handle this issue.
Thank you for raising this important issue. Because the bias comes from the covariance between the regressors and the same GLM was applied to all time points in our analysis, we assume that the inflation would be similar at different time points. Therefore, we calculated the correlation of SC and SR betas ranging from -200 to 0 ms relative to stimulus onset as a baseline (i.e., no SC or SR representation is expected before the stimulus onset) and compared the post-stimulus onset correlation coefficients against this baseline. We hypothesized that if the positively within-trial correlation of SC and SR betas resulted from the simultaneous representation instead of inflation, we should observe significantly higher correlation when compared with the baseline. To examine this hypothesis, we first performed the linear discriminant analysis (Supplementary Fig. 7a) and RSA regression (Supplementary Fig. 7b) on the -200 - 0 ms window relative to stimulus onset. We then calculated the average rbaseline of SC and SR betas on that time window for each participant (group results at each time point are shown in Supplementary Fig. 7c) and computed the relative correlation at each post-stimulus onset time point using (fisher-z (r) - fisher-z (rbaseline)). Finally, we performed a simple t test at the group level on baseline-corrected correlation coefficients with Bonferroni correction. The results (Fig. 6c) showed significantly more positive correlation from 100 - 500 ms post-stimulus onset compared with baseline, supporting our hypothesis that the positive within-trial correlation of SC and SR betas arise from simultaneous representation rather than inflation. The related interpretation was added to page 17 of the revised manuscript.
(4) Are results robust to running response-locked analyses? Especially the EEG-behavior correlation. Could this be driven by different RTs across trials & trial-types? I.e., at 400 ms poststim onset, some trials would be near or at RT/action execution, while others may not be nearly as close, and so EEG features would differ & "predict" RT.
Thanks for this question. We now pair each of the stimulus-locked EEG analysis in the manuscript with response-locked analysis. To control for RT variations among trial types, when using the linear mixed model (LMM) to predict RTs from trial-wise RSA results, we included a separate intercept for each of the eight trial types in SC or SR. Furthermore, at each time point, we only included trials that have not generated a response (for stimulus-locked analysis) or already started (for response-locked analysis). All the results (Fig. 3, 5, 7, 9 in the revised manuscript) are in support of our hypothesis. We added these detailed to page 31 of the revised manuscript.
(5) I suggest providing more explanation about the logic of the subspace decoding method - what trialtypes exactly constitute the different classes, why we would expect this method to capture something useful regarding ISPC, & what this something might be. I felt that the first paragraph of the results breezes by a lot of important logic.
In general, this paper does not seem to be written for readers who are unfamiliar with this particular topic area. If authors think this is undesirable, I would suggest altering the text.
To improve clarity, we revised the first paragraph of the SC and SR association subspace analysis to list the conditions for each of the SC and SR decoders and explain more about how the concept of being separatable can be tested by cross-decoding between SC and SR subspaces. The revised paragraph now reads:
“Prior to testing whether controlled and non-controlled associations were represented simultaneously, we first tested whether the two representations were separable in the EEG data.
In other words, we reorganized the 16 experimental conditions into 8 conditions for SC (4 colors × MC/MI, while collapsing across SR levels) and SR (4 words × 2 possible responses per word, while collapsing across SC levels) associations separately. If SC and SR associations are not separable, it follows that they encode the same information, such that both SC and SR associations can be represented in the same subspace (i.e., by the same information encoded in both associations). For example, because (1) the word can be determined by the color and congruency and (2) the most-likely response can be determined by color and ISPC, the SR association (i.e., association between word and most-likely response) can in theory be represented using the same information as the SC association. On the other hand, if SC and SR associations are separable, they are expected to be represented in different subspaces (i.e., the information used to encode the two associations is different). Notably, if some, but not all, information is shared between SC and SR associations, they are still separable by the unique information encoded. In this case, the SC and SR subspaces will partially overlap but still differ in some dimensions. To summarize, whether SC and SR associations are separable is operationalized as whether the associations are represented in the same subspace of EEG data. To test this, we leveraged the subspace created by the LDA (see Methods). Briefly, to capture the subspace that best distinguishes our experimental conditions, we trained SC and SR decoders using their respective aforementioned 8 experimental conditions. We then projected the EEG data onto the decoding weights of the LDA for each of the SC and SR decoders to obtain its respective subspace. We hypothesized that if SC and SR subspaces are identical (i.e., not separable), SC/SR decoding accuracy should not differ by which subspace (SC or SR) the decoder is trained on. For example, SC decoders trained in SC subspace should show similar decoding performance as SC decoders trained in SR subspace. On the other hand, if SC and SR association representations are in different subspaces, the SC/SR subspace will not encode all information for SR/SC associations. As a result, decoding accuracy should be higher using its own subspace (e.g., decoding SC using the SC subspace) than using the other subspace (e.g., decoding SC using the SR subspace). We used cross-validation to avoid artificially higher decoding accuracy for decoders using their own subspace (see Methods).” (Page 11-12).
We also explicitly tested what information is shared between SC and SR representations (see response to comment #2). Lastly, to help the readers navigate the EEG results, we added a section “Overview of EEG analysis” to summarize the EEG analysis and their relations in the following manner:
“EEG analysis overview. We started by validating that the 16 experimental conditions (8 unique stimuli × MC/MI) were represented in the EEG data. Evidence of representation was provided by above-chance decoding of the experimental conditions (Fig. 2-3). We then examined whether the SC and SR associations were separable (i.e., whether SC and SR associations were different representations of equivalent information). As our results supported separable representations of SC and SR association (Fig. 4-5), we further estimated the temporal dynamics of each representation within a trial using RSA. This analysis revealed that the temporal dynamics of SC and SR association representations overlapped (Fig. 6a-b, Fig. 7a-b). To explore the potential reason behind the temporal overlap of the two representations, we investigated whether SC and SR associations were represented simultaneously as part of the task representation, independently from each other, or competitively/exclusively (e.g., on some trials only SC association was represented, while on other trials only SR association was represented). This was done by assessing the correlation between the strength of SC and SR representations across trials (Fig. 6c, Fig. 7c). Lastly, we tested how SC and SR representations facilitated performance (Fig.8-9).” (Page 8-9).
Minor suggestions:
(6) I'd suggest using single-trial RSA beta coefficients, not t-values, as they can be more stable (it's a t-value based on 16 observations against 9 or so regressors.... the SE can be tiny).
Thank you for your suggestion. To choose between using betas and t-values, we calculate the proportion of outliers (defined as values beyond mean ± 5 SD) for each predictor of the design matrix and each subject. We found that outliers were less frequent for t-values than for beta coefficients (t-values: mean = 0.07%, SD = 0.009%; beta-values: mean = 0.19%, SD = 0.033%). Thus, we decided to stay with t-values.
(7) Instead of prewhitening the RTs before the HLM with drift terms, try putting those in the HLM itself, to avoid two-stage regression bias.
Thank you for your suggestion. Because our current LMM included each of the eight trial types in SC or SR as separate predictors with their own intercepts (as mentioned above), adding regressors of trial number and mini blocks (1-100 blocks) introduced collinearity (as ISPC flipped during the experiment). We therefore excluded these regressors from the current LMM (Page 31).
(8) The text says classical MDS was performed on decoding *accuracy* - is this accurate?
We now clarify in the manuscript that it is the decoders’ probabilistic classification results (Page 28).
(9) At a few points, it was claimed that a negative correlation between SC and SR would be expected within single trials, if the two were temporally dissociable. Wouldn't it also be possible that they are not correlated/orthogonal?
We agree with the reviewer and revised the null hypothesis in the cross-trial correlation analysis to include no correlation as SC and SR association representations may be independent from each other (Page 17, 22).
Reviewer #2 (Public review):
Summary:
In this EEG study, Huang et al. investigated the relative contribution of two accounts to the process of conflict control, namely the stimulus-control association (SC), which refers to the phenomenon that the ratio of congruent vs. incongruent trials affects the overall control demands, and the stimulus-response association (SR), stating that the frequency of stimulusresponse pairings can also impact the level of control. The authors extended the Stroop task with novel manipulation of item congruencies across blocks in order to test whether both types of information are encoded and related to behaviour. Using decoding and RSA, they showed that the SC and SR representations were concurrently present in voltage signals, and they also positively co-varied. In addition, the variability in both of their strengths was predictive of reaction time. In general, the experiment has a solid design, but there are some confounding factors in the analyses that should be addressed to provide strong support for the conclusions.
Strengths:
(1) The authors used an interesting task design that extended the classic Stroop paradigm and is potentially effective in teasing apart the relative contribution of the two different accounts regarding item-specific proportion congruency effect, provided that some confounds are addressed.
(2) Linking the strength of RSA scores with behavioural measures is critical to demonstrating the functional significance of the task representations in question.
Thank you for your positive feedback. We hope our responses below address your concerns.
Weakness:
(1) While the use of RSA to model the decoding strength vector is a fitting choice, looking at the RDMs in Figure 7, it seems that SC, SR, ISPC, and Identity matrices are all somewhat correlated. I wouldn't be surprised if some correlations would be quite high if they were reported. Total orthogonality is, of course, impossible depending on the hypothesis, but from experience, having highly covaried predictors in a regression can lead to unexpected results, such as artificially boosting the significance of one predictor in one direction, and the other one to the opposite direction. Perhaps some efforts to address how stable the timed-resolved RSA correlations for SC and SR are with and without the other highly correlated predictors will be valuable to raising confidence in the findings.
Thank you for this important point. The results of proportion of variability explained shown in the Author response table 1 below, indicated relatively higher correlation of SC/SR with Color and Identity. We agree that it is impossible to fully orthogonalize them. To address the issue of collinearity, we performed a control RSA by removing predictors highly correlated with others. Specifically, we calculated the variance inflation factor (VIF) for each predictor. The Identity predictor had a high VIF of 5 and was removed from the RSA. All other predictors had VIFs < 4 and were kept in the RSA. The results (Supplementary Fig. 6) showed patterns similar to the results with the Identity predictor, suggesting that the findings are not significantly influenced by collinearity. We have added the interpretation to page 17 of the revised manuscript.
Author response table 1.
Proportion of variability explained (r2) of RSA predictors.
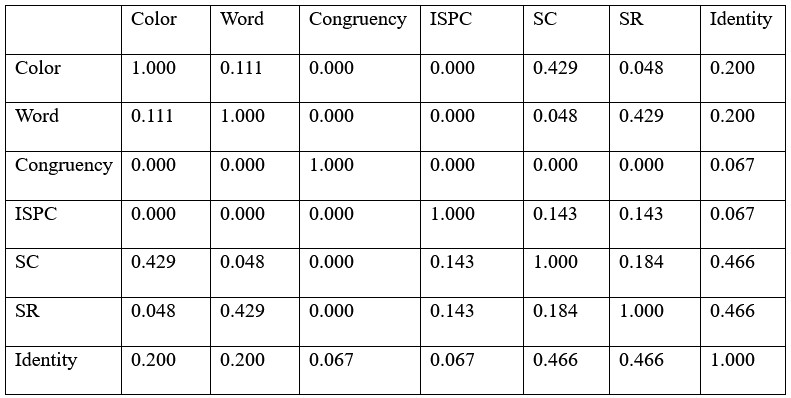
(2) In "task overview", SR is defined as the word-response pair; however, in the Methods, lines 495-496, the definition changed to "the pairing between word and ISPC" which is in accordance with the values in the RDMs (e.g., mccbb and mcirb have similarity of 1, but they are linked to different responses, so should they not be considered different in terms of SR?). This needs clarification as they have very different implications for the task design and interpretation of results, e.g., how correlated the SC and SR manipulations were.
Thank you for pointing out this important issue with how our operationalization captures the concept in questions. In the revised manuscript, we clarified the stimulus-response (SR) association is the link between the word and the most-likely response (i.e., not necessarily the actual response on the current trial). This association is likely to be encoded based on statistical learning over several trials. On each trial, the association is updated based on the stimulus and the actual response. Over multiple trials, the accumulated association will be driven towards the most-common (i.e., most-likely) response. In our ISPC manipulation, a color is presented in mostly congruent/incongruent (MC/MI) trials, which will also pair a word with a most-likely response. For example, if the color blue is MC, the color blue, which leads to the response blue, will co-occur with the word blue with high frequency. In other words, the SR association here is between the word blue and the response blue. As the actual response is not part of the SR association, in the RDM two trial types with different responses may share the same SR association, as long as they share the same word and the same ISPC manipulation, which, by the logic above, will produce the same most-likely response. These clarifications have been added to page 4 and 29 of the revised manuscript.
In the revised manuscript (Page 17), we addressed how much the correlated SC and SR predictors in the RDM could affect the correlation analysis between SC and SR association representation strength. Specifically, we conducted the RSA using the same GLM on EEG data prior to stimulus onset (Supplementary Fig. 7a-b). As no SC and SR associations are expected to be present before stimulus onset, the correlation between SC and SR representation would serve as a baseline of inflation due to correlated predictors in the GLM (Supplementary Fig. 7c, also see comment #3 of R1). The SC-SR correlation coefficients following stimulus onset was then compared to the baseline to control for potential inflation (Fig. 6c). Significantly above-baseline correlation was still observed between ~100-500 ms post-stimulus onset, providing support for the hypothesis that SC and SR are encoded in the same task representation.
Minor suggestions:
(3) Overall, I find that calling SC-controlled and SR-uncontrolled representations unwarranted. How is the level controlledness defined? Both are essentially types of statistical expectation that provide contextual information for the block of tasks. Is one really more automatic and requires less conscious processing than the other? More background/justification could be provided if the authors would like to use these terms.
Following your advice, we have added more discussion on how controlledness is conceptualized in this work and in the literature, which reads:
“We consider SC and SR as controlled and uncontrolled respectively based on the literature investigating the mechanism of ISPC effect. The SC account posits that the ISPC effect results from conflict and involves conflict adaptation, which requires the regulation of attention or control (Bugg & Hutchison, 2013; Bugg et al., 2011; Schmidt, 2018; Schmidt & Besner, 2008). On the other hand, the SR account argues that ISPC effect does not require conflict adaptation but instead reflects contingency leaning. That is, the response can be directly retrieved from the association between the stimulus and the most-likely response without top-down regulation of attention or control. As more empirical evidence emerged, researchers advocating control view began to acknowledge the role of associative learning in cognitive control regarding the ISPC effect (Abrahamse et al., 2016). SC association has been thought to include both automatic that is fast and resource saving and controlled processes that is flexible and generalizable (Chiu, 2019). Overall, we do not intend to claim that SC is entirely controlled or SR is completely automatic. We use SC-controlled and SR-uncontrolled representations to align with the original theoretical motivation and to highlight the conceptual difference between SC and SR associations.” (Page 24-25)
(4) Figures 3c and d: the figures could benefit from more explanation of what they try to show to the readers. Also for 3d, the dimensions were aligned with color sets and congruencies, but word identities were not linearly separable, at least for the first 3 axes. Shouldn't one expect that words can be decoded in the SR subspace if word-response pairs were decodable (e.g., Figure 3b)?
Thank you for the insightful observation. We now clarified that Fig. 3c and d in the original manuscript (Fig. 4c and d in the current manuscript) aim to show how each of the 8 trial types in the SC and SR subspaces are represented. The MDS approach we used for visualization tries to preserve dissimilarity between trial types when projecting from data from a high dimensional to a low dimensional space. However, such projection may also make patterns linearly separatable in high dimensional space not linearly separatable in low dimensional space. For example, if the word blue has two points (-1, -1) and (1, 1) and the word red has two points (-1, 1) and (1, -1), they are not linearly separatable in the 2D space. Yet, if they are projected from a 3D space with coordinates of (-1, -1, -0.1), (1, 1, -0.1), (-1, 1, 0.1) and (1, -1, 0.1), the two words can be linearly separatable using the 3rd dimension. Thus, a better way to test whether word can be linearly separated in SR subspace is to perform RSA on the original high dimensional space. We performed the RSA with word (Supplementary Fig. 2) on the SR decoder trained on the SR subspace. Note that in Fig. 3c and d of the original script (Fig. 4c and d in the current manuscript) there are two pairs of words that are not linearly separable: red-blue and yellow-green. Thus, we specifically tested the separability within the two pairs using the one predictor for each pair, as shown in Supplementary Fig. 2. The results showed that within both word pairs individual words were presented above chance level (Supplementary Fig. 3). Considering that the decoders are linear, this finding indicates linear separability of the word pairs in the original SR subspace. The clarification has been added to page 13 (the end of the second paragraph) of the revised manuscript.
References
Abrahamse, E., Braem, S., Notebaert, W., & Verguts, T. (2016). Grounding cognitive control in associative learning. Psychological Bulletin, 142(7), 693-728.doi:10.1037/bul0000047.
Bugg, J. M., & Hutchison, K. A. (2013). Converging evidence for control of color-word Stroop interference at the item level. Journal of Experimental Psychology:Human Perception and Performance, 39(2), 433-449. doi:10.1037/a0029145.
Bugg, J. M., Jacoby, L. L., & Chanani, S. (2011). Why it is too early to lose control in accounts of item-specific proportion congruency effects. Journal of Experimental Psychology: Human Perception and Performance, 37(3), 844-859. doi:10.1037/a0019957.
Chiu, Y.-C. (2019). Automating adaptive control with item-specific learning. In Psychology of Learning and Motivation (Vol. 71, pp. 1-37).
Schmidt, J. R. (2018). Evidence against conflict monitoring and adaptation: An updated review. Psychonomic Bulletin & Review, 26(3), 753-771. doi:10.3758/s13423018-1520-z.
Schmidt, J. R., & Besner, D. (2008). The Stroop effect: Why proportion congruent has nothing to do with congruency and everything to do with contingency. Journal of Experimental Psychology: Learning, Memory, and Cognition, 34(3), 514-523. doi:10.1037/0278-7393.34.3.514.
-
-
-
-
eLife Assessment
This useful study uses creative scalp EEG decoding methods to attempt to demonstrate that two forms of learned associations in a Stroop task are dissociable, despite sharing similar temporal dynamics. However, the evidence supporting the conclusions is incomplete due to concerns with the experimental design and methodology. This paper would be of interest to researchers studying cognitive control and adaptive behavior, if the concerns raised in the reviews can be addressed satisfactorily.
-
Reviewer #1 (Public review):
Summary:
This study focuses on characterizing the EEG correlates of item-specific proportion congruency effects. In particular, two types of learned associations are characterized. One being associations between stimulus features and control states (SC), and the other being stimulus features and responses (SR). Decoding methods are used to identify SC and SR correlates and to determine whether they have similar topographies and dynamics.
The results suggest SC and SR associations are simultaneously coactivated and have shared topographies, with the inference being that these associations may share a common generator.
Strengths:
Fearless, creative use of EEG decoding to test tricky hypotheses regarding latent associations.
Nice idea to orthogonalize the ISPC condition (MC/MI) from stimulus features.
Weaknesses:
Reviewer #1 (Public review):
Summary:
This study focuses on characterizing the EEG correlates of item-specific proportion congruency effects. In particular, two types of learned associations are characterized. One being associations between stimulus features and control states (SC), and the other being stimulus features and responses (SR). Decoding methods are used to identify SC and SR correlates and to determine whether they have similar topographies and dynamics.
The results suggest SC and SR associations are simultaneously coactivated and have shared topographies, with the inference being that these associations may share a common generator.
Strengths:
Fearless, creative use of EEG decoding to test tricky hypotheses regarding latent associations.
Nice idea to orthogonalize the ISPC condition (MC/MI) from stimulus features.
Weaknesses:
(1) I'm relatively concerned that these results may be spurious. I hope to be proven wrong, but I would suggest taking another look at a few things.
While a nice idea in principle, the ISPC manipulation seems to be quite confounded with the trial number. E.g., color-red is MI only during phase 2, and is MC primarily only during Phase 3 (since phase 1 is so sparsely represented). In my experience, EEG noise is highly structured across a session and easily exploited by decoders. Plus, behavior seems quite different between Phase 2 and Phase 3. So, it seems likely that the classes you are asking the decoder to separate are highly confounded with temporally structured noise.
I suggest thinking of how to handle this concern in a rigorous way. A compelling way to address this would be to perform "cross-phase" decoding, however I am not sure if that is possible given the design.
The time courses also seem concerning. What are we to make of the SR and SC timecourses, which have aggregate decoding dynamics that look to be <1Hz?
Some sanity checks would be one place to start. Time courses were baselined, but this is often not necessary with decoding; it can cause bias (10.1016/j.jneumeth.2021.109080), and can mask deeper issues. What do things look like when not baselined? Can variables be decoded when they should not be decoded? What does cross-temporal decoding look like - everything stable across all times, etc.?
(2) The nature of the shared features between SR and SC subspaces is unclear.
The simulation is framed in terms of the amount of overlap, revealing the number of shared dimensions between subspaces. In reality, it seems like it's closer to 'proportion of volume shared', i.e., a small number of dominant dimensions could drive a large degree of alignment between subspaces.
What features drive the similarity? What features drive the distinctions between SR and SC? Aside from the temporal confounds I mentioned above, is it possible that some low-dimensional feature, like EEG congruency effect (e.g., low-D ERPs associated with conflict), or RT dynamics, drives discriminability among these classes? It seems plausible to me - all one would need is non-homogeneity in the size of the congruency effect across different items (subject-level idiosyncracies could contribute: 10.1016/j.neuroimage.2013.03.039).
(3) The time-resolved within-trial correlation of RSA betas is a cool idea, but I am concerned it is biased. Estimating correlations among different coefficients from the same GLM design matrix is, in general, biased, i.e., when the regressors are non-orthogonal. This bias comes from the expected covariance of the betas and is discussed in detail here (10.1371/journal.pcbi.1006299). In short, correlations could be inflated due to a combination of the design matrix and the structure of the noise. The most established solution, to cross-validate across different GLM estimations, is unfortunately not available here. I would suggest that the authors think of ways to handle this issue.
(4) Are results robust to running response-locked analyses? Especially the EEG-behavior correlation. Could this be driven by different RTs across trials & trial-types? I.e., at 400 ms post-stim onset, some trials would be near or at RT/action execution, while others may not be nearly as close, and so EEG features would differ & "predict" RT.
(5) I suggest providing more explanation about the logic of the subspace decoding method - what trialtypes exactly constitute the different classes, why we would expect this method to capture something useful regarding ISPC, & what this something might be. I felt that the first paragraph of the results breezes by a lot of important logic.
In general, this paper does not seem to be written for readers who are unfamiliar with this particular topic area. If authors think this is undesirable, I would suggest altering the text.
-
Reviewer #2 (Public review):
Summary:
In this EEG study, Huang et al. investigated the relative contribution of two accounts to the process of conflict control, namely the stimulus-control association (SC), which refers to the phenomenon that the ratio of congruent vs. incongruent trials affects the overall control demands, and the stimulus-response association (SR), stating that the frequency of stimulus-response pairings can also impact the level of control. The authors extended the Stroop task with novel manipulation of item congruencies across blocks in order to test whether both types of information are encoded and related to behaviour. Using decoding and RSA, they showed that the SC and SR representations were concurrently present in voltage signals, and they also positively co-varied. In addition, the variability in both of their …
Reviewer #2 (Public review):
Summary:
In this EEG study, Huang et al. investigated the relative contribution of two accounts to the process of conflict control, namely the stimulus-control association (SC), which refers to the phenomenon that the ratio of congruent vs. incongruent trials affects the overall control demands, and the stimulus-response association (SR), stating that the frequency of stimulus-response pairings can also impact the level of control. The authors extended the Stroop task with novel manipulation of item congruencies across blocks in order to test whether both types of information are encoded and related to behaviour. Using decoding and RSA, they showed that the SC and SR representations were concurrently present in voltage signals, and they also positively co-varied. In addition, the variability in both of their strengths was predictive of reaction time. In general, the experiment has a solid design, but there are some confounding factors in the analyses that should be addressed to provide strong support for the conclusions.
Strengths:
(1) The authors used an interesting task design that extended the classic Stroop paradigm and is potentially effective in teasing apart the relative contribution of the two different accounts regarding item-specific proportion congruency effect, provided that some confounds are addressed.
(2) Linking the strength of RSA scores with behavioural measures is critical to demonstrating the functional significance of the task representations in question.
Weakness:
(1) While the use of RSA to model the decoding strength vector is a fitting choice, looking at the RDMs in Figure 7, it seems that SC, SR, ISPC, and Identity matrices are all somewhat correlated. I wouldn't be surprised if some correlations would be quite high if they were reported. Total orthogonality is, of course, impossible depending on the hypothesis, but from experience, having highly covaried predictors in a regression can lead to unexpected results, such as artificially boosting the significance of one predictor in one direction, and the other one to the opposite direction. Perhaps some efforts to address how stable the timed-resolved RSA correlations for SC and SR are with and without the other highly correlated predictors will be valuable to raising confidence in the findings.
(2) In "task overview", SR is defined as the word-response pair; however, in the Methods, lines 495-496, the definition changed to "the pairing between word and ISPC" which is in accordance with the values in the RDMs (e.g., mccbb and mcirb have similarity of 1, but they are linked to different responses, so should they not be considered different in terms of SR?). This needs clarification as they have very different implications for the task design and interpretation of results, e.g., how correlated the SC and SR manipulations were.
-
Adaptive behavior is guided by integrated representations of controlled and non-controlled information https://www.biorxiv.org/content/10.1101/2025.08.07.669231v1
-
Adaptive behavior is guided by integrated representations of controlled and non-controlled information https://www.biorxiv.org/content/10.1101/2025.08.07.669231v1
-